



Agricultural intensification is one of the leading drivers of global biodiversity loss. Assessing its ecological impacts requires more than just measuring species richness; incorporating functional diversity allows for deeper insight into changes in community structure and ecosystem functioning. Amphibians are sensitive to environmental change, making them ideal indicators of ecosystem health. In this study, we examined how agricultural management influences the taxonomic and functional diversity of anuran communities in the Brazilian Pampa. We surveyed anurans in 26 ponds across 16 family farms (nine organics and seven conventional), sampled three times during the 2023–2024 breeding seasons. Diversity metrics were assessed at both the pond and farming levels, incorporating local habitat features and landscape composition at multiple spatial scales. Results showed that organic agroecosystems supported higher species richness at the pond scale, although functional diversity did not differ between management types at this level. In contrast, at the agroecosystem scale, organic farming supported higher functional diversity than conventional systems. Additionally, we found a significant interaction between management type and surrounding forest cover: organic farming adjacent to forest patches had the highest diversity values. Our findings highlight the importance of integrating sustainable agricultural practices with the conservation of natural landscape elements. Promoting organic farming alongside the preservation of native habitats can help mitigate the negative effects of intensification and enhance biodiversity in agricultural landscapes.

Agricultural intensification is one of the main drivers of biodiversity loss in worldwide (Flynn et al., 2009; Tuck et al., 2014). Understanding how different farming systems influence biodiversity has become essential for reconciling food production with conservation objectives (Tuck et al., 2014). In this context, organic farming has been proposed as a more biodiversity-friendly alternative to conventional agriculture, as it avoids synthetic fertilizers and pesticides, promotes crop rotation, and generally involves lower land-use intensity, thereby potentially mitigating negative impacts on wildlife while maintaining agricultural productivity (Katayama et al., 2019; Tuck et al., 2014).
The Pampa biome, one of the most threatened ecosystems in Brazil, is dominated by natural grasslands but also includes forests, savannas, palm groves, rocky outcrops, dunes, wetlands, and water bodies (Andrade et al., 2023). In southern Rio Grande do Sul, the Pampa is regionally and continentally important for family farming, legally defined in Brazil as agricultural systems based on family labor and diversified land use (Cicconeto and Verdum, 2012). In this landscape, biodiversity conservation depends not only on the type of agricultural management but also on the structure and composition of the surrounding landscape matrix (Iop et al., 2020).
Amphibians are among the vertebrate groups most threatened vertebrates globally (Harfoot et al., 2021). Their complex life cycles, low dispersal capacity, and dependence on both aquatic and terrestrial habitats make anurans particularly suitable ecological models for assessing the effects of agricultural intensification (Collins and Fahrig, 2017). Most anuran species rely on waterbodies for breeding and larval development, while the surrounding terrestrial environment is essential for foraging, shelter, and dispersal (Moreira et al., 2020). Consequently, anuran communities are structured by processes operating at multiple spatial scales, including local characteristics of breeding sites, such as pond area, depth, vegetation structure, and the presence of predators, as well as landscape attributes that influence habitat availability, connectivity, and movement among ponds (Queiroz et al., 2015; Moreira et al., 2020).
In agricultural contexts, conventional farming practices have been consistently associated with reduced anuran richness and abundance, whereas organic systems often mitigate these effects (Maltchik et al., 2017; Moreira et al., 2014). However, responses to agricultural management are not uniform and may strongly depend on landscape context (Agostini et al., 2021). The amount of native vegetation, habitat heterogeneity, and the spatial arrangement of aquatic and terrestrial habitats can mediate the effectiveness of farming practices in conserving amphibian diversity (Collins and Fahrig, 2017). In grassland-dominated farming such as the Pampa, where breeding habitats are often artificial and embedded within managed matrices, disentangling the relative roles of local habitat conditions and surrounding landscape structure is particularly important (Moreira et al., 2020; Oro et al., 2024).
Although many studies evaluating the impacts of agricultural intensification on amphibians have focused on taxonomic diversity, other dimensions of biodiversity, such as functional diversity, remain comparatively understudied in agricultural landscapes (Pereyra et al., 2018). Functional diversity, defined as the range and distribution of functional traits within a community (Violle et al., 2007), provides insights into community assembly processes and reflects the capacity of communities to respond to environmental change (de Bello et al., 2021). Traits related to body size, reproductive mode, habitat use, and dispersal ability are particularly relevant for amphibians in agroecosystems, as they influence species’ sensitivity to habitat alteration (Pereyra et al., 2018). Moreover, community composition analyses can reveal whether different management systems promote distinct assemblages or lead to biotic homogenization across the landscape (Oro et al., 2024; Preuss et al., 2024).
In this study, we classified farming using pesticides, and high land-use intensity as conventional, whereas organic farming relied on natural alternatives for pest and soil management, lower chemical inputs, and reduced land-use intensity (Carvalho et al., 2025). Importantly, organic management in the study area does not inherently imply greater native vegetation cover around ponds, allowing us to evaluate management effects independently from landscape composition. Both farming systems are embedded within heterogeneous agricultural landscapes characterized by a mosaic of grasslands, forest patches, crops, and artificial ponds, which serve as key breeding habitats for amphibians (Iop et al., 2020).
We aimed to compare taxonomic, functional, and beta diversity, as well as community composition of anurans between organic and conventional agroecosystems in the Brazilian Pampa. Additionally, we evaluated how local habitat characteristics of ponds and landscape composition at different spatial scales influence diversity patterns and community assembly. We hypothesized that organic agroecosystems would support higher taxonomic and functional diversity and distinct community composition compared to conventional systems, although functional composition may remain similar if assemblages are functionally redundant. We further expected that higher native vegetation cover in the surrounding landscape would positively influence diversity metrics.
Materials and methodsStudy areaThe study was conducted in 16 agroecosystems located in the Rio Grande do Sul state, Brazil, within the Serra do Sudeste physiographic region, part of the Pampa biome. The landscape is characterized by shallow, rocky soils and predominantly rugged relief. Natural grasslands occur in a mosaic pattern, interspersed with fragments of semi-deciduous seasonal forest (Overbeck et al., 2015).
Seven farms were managed under conventional agricultural practices, whereas nine adopted organic farming. The main agricultural activities included fruit cultivation, particularly peaches, oranges, and guavas, as well as annual crops such as beans, corn, soybeans, and tobacco.
Anuran samplingAnuran surveys were conducted during the reproductive season, with each farming sampled twice in spring (October–November 2023) and once in summer (March 2024), following Both et al. (2008). Because all anuran species occurring in the region depend on water bodies for reproduction, all artificial ponds within each agroecosystem were surveyed to maximize detection probability.
Farms were spaced 1–20 km apart. A total of 26 ponds were sampled, with inter-pond distances ranging from 80 to 520 m. Eleven ponds were located in conventional farming and 15 in organic ones. Surveys were conducted from 30 min after sunset until 23:00 h using visual and acoustic encounter surveys, with each pond surveyed for 30 min by two observers (i.e., 60 person-minutes per pond; Scott and Woodward, 1994). During each survey, observers divided the pond perimeter and actively walked along the shoreline to maximize spatial coverage. Sampling effort was standardized across ponds regardless of pond size or structural complexity; therefore, survey duration was kept constant among sampling units. Visual and acoustic methods were applied simultaneously by two observers during periods of peak amphibian activity. Because many species recorded in the study area exhibit fossorial habits or cryptic behavior that prevents reliable abundance estimation, we used incidence-based data in all analyses.
Characteristics of the ponds in the farmsFor each pond, we measured a set of local habitat variables known to influence anuran occurrence (Moreira et al., 2020; Iop et al., 2020). Pond surface area was measured in the field for small ponds and estimated from high-resolution satellite imagery (Google Earth) for larger ponds. Maximum depth was measured at five points per pond using a graduated 1-m ruler. Physicochemical variables included pH and electrical conductivity, measured with a Hanna VCx3 multiparameter device. Aquatic and marginal vegetation cover and fish presence were visually estimated during field surveys.
To reduce collinearity among pond-level variables and summarize local environmental variation, we performed a Principal Coordinate Analysis (PCoA) using a Gower distance matrix. The first two ordination axes were retained and used as synthetic descriptors of pond characteristics in subsequent analyses (Fig. S2).
Characteristics of the landscape in different scalesLandscape composition was quantified at two spatial scales to capture ecological processes operating at different levels. At the pond level, landscape variables were measured within a 200 m radius centered on each pond, reflecting the spatial scale at which local habitat structure and short-distance movements influence amphibian occurrence (Preuss et al., 2024). At the farming level, landscape variables were quantified within a 500 m radius centered on the farms centroid, representing broader landscape context and habitat availability in the region (Iop et al., 2020; Moreira et al., 2020; Oro et al., 2024). The land-cover data were obtained from MapBiomas Collection 9.0 (2023) using Google Earth Engine. We quantified the proportions of forest, silviculture, grassland, and farmland within each buffer. Due to strong correlations among land-cover variables, only forest and silviculture cover were retained as predictors for subsequent analysis (Fig. S4 and Fig. S5).
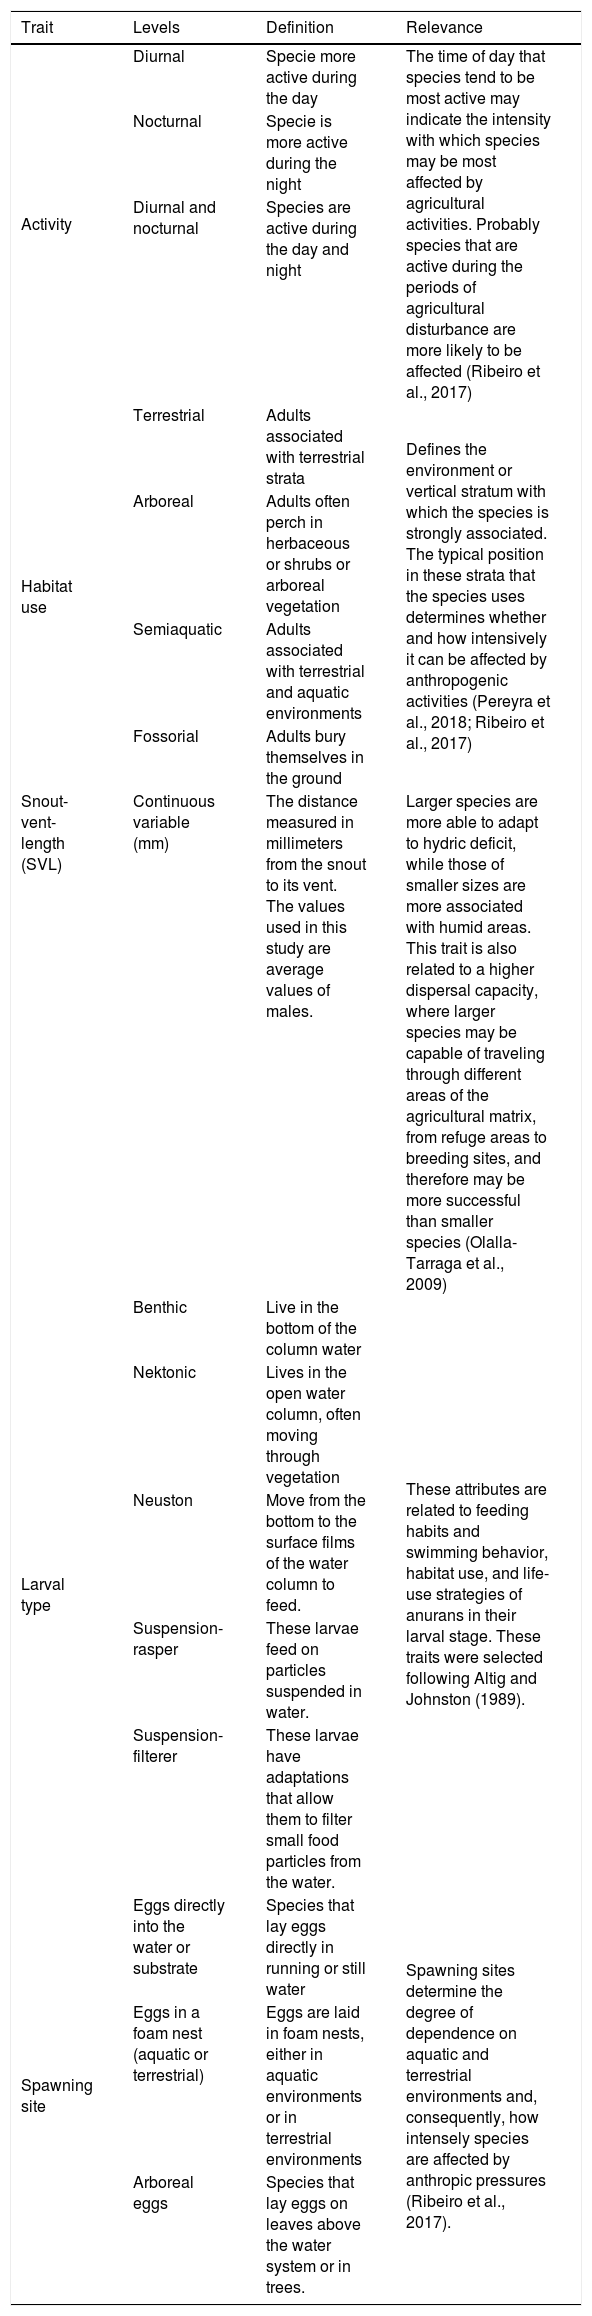
Anuran traitsFunctional trait data were compiled from the literature. Selected traits represent key aspects of the anuran life cycle and ecological strategies. These traits are expected to influence species’ responses to habitat alteration in farming. A detailed description of traits and their ecological relevance is provided in Table 1.
Definitions and relevance of anuran traits used in functional analyses.
| Trait | Levels | Definition | Relevance |
|---|---|---|---|
| Activity | Diurnal | Specie more active during the day | The time of day that species tend to be most active may indicate the intensity with which species may be most affected by agricultural activities. Probably species that are active during the periods of agricultural disturbance are more likely to be affected (Ribeiro et al., 2017) |
| Nocturnal | Specie is more active during the night | ||
| Diurnal and nocturnal | Species are active during the day and night | ||
| Habitat use | Terrestrial | Adults associated with terrestrial strata | Defines the environment or vertical stratum with which the species is strongly associated. The typical position in these strata that the species uses determines whether and how intensively it can be affected by anthropogenic activities (Pereyra et al., 2018; Ribeiro et al., 2017) |
| Arboreal | Adults often perch in herbaceous or shrubs or arboreal vegetation | ||
| Semiaquatic | Adults associated with terrestrial and aquatic environments | ||
| Fossorial | Adults bury themselves in the ground | ||
| Snout-vent-length (SVL) | Continuous variable (mm) | The distance measured in millimeters from the snout to its vent. The values used in this study are average values of males. | Larger species are more able to adapt to hydric deficit, while those of smaller sizes are more associated with humid areas. This trait is also related to a higher dispersal capacity, where larger species may be capable of traveling through different areas of the agricultural matrix, from refuge areas to breeding sites, and therefore may be more successful than smaller species (Olalla-Tarraga et al., 2009) |
| Larval type | Benthic | Live in the bottom of the column water | These attributes are related to feeding habits and swimming behavior, habitat use, and life-use strategies of anurans in their larval stage. These traits were selected following Altig and Johnston (1989). |
| Nektonic | Lives in the open water column, often moving through vegetation | ||
| Neuston | Move from the bottom to the surface films of the water column to feed. | ||
| Suspension-rasper | These larvae feed on particles suspended in water. | ||
| Suspension-filterer | These larvae have adaptations that allow them to filter small food particles from the water. | ||
| Spawning site | Eggs directly into the water or substrate | Species that lay eggs directly in running or still water | Spawning sites determine the degree of dependence on aquatic and terrestrial environments and, consequently, how intensely species are affected by anthropic pressures (Ribeiro et al., 2017). |
| Eggs in a foam nest (aquatic or terrestrial) | Eggs are laid in foam nests, either in aquatic environments or in terrestrial environments | ||
| Arboreal eggs | Species that lay eggs on leaves above the water system or in trees. |
The presence of phylogenetic signal in ecological traits can inflate type I error in ecological analyses (Harvey and Pagel, 1991). To account for this, we repeated all analyses after controlling for phylogenetic signal in trait data and compared them with those obtained using raw trait values. We used a consensus phylogeny for anurans based on Jetz and Pyron (2018), pruned to include only species occurring in the Pampa biome. Nine species names were updated according to current taxonomy. Three species absent from the original tree (Julianus fontanarrosae, Odontophrynus reigi, and Leptodactylus luctator) were manually inserted as sister taxa to closely related species (Scinax pinima, Odontophrynus cordobae, and Leptodactylus latrans, respectively; Magalhães et al., 2020; Rosset et al., 2021; Araujo-Vieira et al., 2023). Although inserting taxa not present in the original phylogeny may introduce some uncertainty in tree topology and branch lengths, these insertions were restricted to terminal nodes and therefore are not expected to substantially affect PVR results. Previous studies have shown that terminal polytomies generally have negligible effects on phylogenetic signal estimates (Münkemüller et al., 2012). We then performed phylogenetic eigenvector regression (PVR; Diniz-Filho et al., 1998) on both binary and continuous traits. Phylogenetic eigenvectors were extracted from species distance matrices using principal coordinates analysis and selected for each trait using Moran’s I criterion (Diniz-Filho et al., 2012). Residuals from the resulting regression models, representing trait variation independent of phylogeny (Diniz-Filho et al., 2011), were subsequently used to recalculate all functional diversity and functional composition metrics, allowing direct comparison with analyses based on raw trait values. All procedures were implemented in R using the function PVRdecomp from the PVR package (R Core Team, 2024).
Species richness and functional diversity in the pondsSpecies richness (SR) and functional diversity (FD) were calculated for each pond. Functional diversity was estimated using the Petchey and Gaston (2006) index, which quantifies the sum of branch lengths in a functional dendrogram based on trait dissimilarities among species. We converted the functional trait matrix into a distance matrix using the Gower distance, suitable for analyzing mixed variables (continuous and categorical). Then, we constructed a functional dendrogram using the unweighted pair groups method with arithmetic mean (UPGMA).
We calculated the standardized effect size of FD (SES.FD) to account for SR effects. SES.FD was computed using 999 null communities generated by random sampling from the regional species pool of the Brazilian Pampa (N = 59 species; Andrade et al., 2023). In each simulation, species richness was constrained to match the observed richness of each sampling unit, while species identities were randomly drawn without replacement and with equal probability of occurrence. Functional dendrograms were constructed using Gower distances among species traits and the UPGMA clustering algorithm. SES.FD was calculated as:
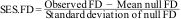
Positive or negative SES.FD values indicate functional diversity higher or lower than expected under the null model, respectively. Additional details on species pool composition are provided in Supplementary Material S1.
Statistical analysesAll statistical analyses were performed in R software (R Core Team, 2024). Sampling sufficiency for each agroecosystem type was assessed using sample coverage analysis based on presence–absence data, implemented with the iNEXT package (Chao et al., 2016).
To assess pond-level diversity patterns, we fitted generalized linear mixed models (GLMMs) relating SR and SES.FD to local and landscape predictors. Fixed effects included agricultural management type, pond characteristics (summarized by the first two PCoA axes), and landscape composition within a 200 m radius. Farming identity was included as a random effect to account for the non-independence of ponds within the same farm.
To describe functional composition, we conducted a PCoA on a Gower distance matrix of functional traits. Community-weighted means (CWMs) were calculated for each ordination axis using incidence-based data, such that each species present in a pond contributed equally to the community mean (de Bello et al., 2021).
Because CWM values can be influenced by species composition, we used a permutation-based approach to test CWM–environment relationships while accounting for species turnover (Peres-Neto et al., 2017). We adapted the cwm.sig function (Duarte et al., 2018), which performs two permutation tests: site shuffling, assessing environmental effects on species distribution, and trait shuffling, evaluating CWM–environment associations independent of species composition.
Differences in taxonomic and functional composition among ponds under organic and conventional farming were assessed using PERMANOVA (Anderson, 2001), with 999 permutations. Taxonomic beta diversity and its turnover and nestedness components were calculated following the additive partitioning framework of Baselga (2012), using Jaccard dissimilarity.
Functional beta diversity was quantified by representing species’ trait spaces as multidimensional hypervolumes (Blonder, 2018). Turnover and nestedness components were also estimated using Jaccard dissimilarity for functional data.
Species richness and functional diversity in the agroecosystemsTo assess species richness and functional diversity at the farming level, species occurrences were pooled across ponds within each farm, and SR and SES.FD were calculated using the same procedures described above. These metrics were modeled as functions of agricultural management type and landscape composition within a 500 m radius.
Generalized Linear Models (GLMs) were used to test for interactions between management type and landscape features. For all analyses, we evaluated whether the residuals were spatially structured based on Moran’s I autocorrelation test.
ResultsWe recorded 20 native anuran species and one exotic Aquarana catesbeiana in the study area, with sampling coverage above 90% (Fig. S1). Organic farming hosted 20 species, compared to 17 in conventional agroecosystems. Boana faber, Leptodactylus mystacinus, Limnomedusa macroglossa, and Rhinella achavali occurred only in organic systems, while Ololygon berthae was exclusive to conventional ones (Table S1).
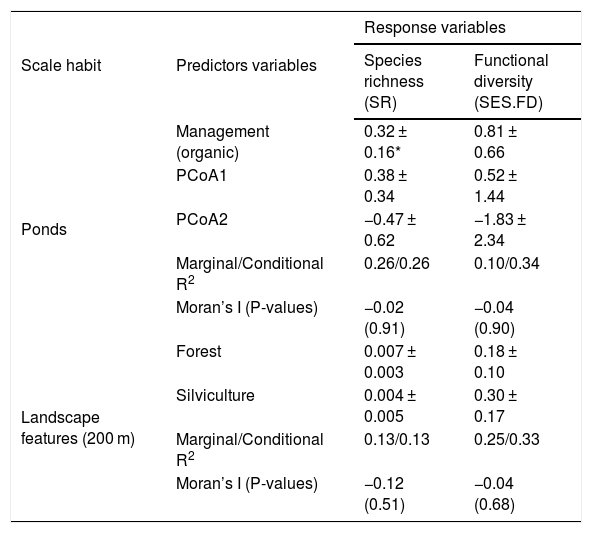
No spatial autocorrelation was detected in model residuals (Tables 2–4). The results of the principal coordinates analysis (PCoA) on the measured variables characterizing the ponds indicate that the first axis accounts for 65.76% of the total variation, while the second axis explains an additional 20.62% of the total environmental variation (Fig. S2). Ponds with positive values on the first axis (hereafter referred to as PCoA1) are associated with higher vegetation cover on their surface, whereas ponds with negative PCoA1 values tend to have a greater presence of fish (Fig. S2). In contrast, the second axis (hereafter referred to as PCoA2) shows that positive values are linked to ponds with larger surface area, while negative PCoA2 values correspond to deeper ponds (Fig. S2).
GLMM relating species richness and functional diversity (SES.FD) of anurans to management type and environmental conditions, summarized in the first two axes of the principal component coordinates (pond characteristics: PCoA1 and PCoA2) and the landscape features in farms in southern Brazil.
| Scale habit | Predictors variables | Response variables | |
|---|---|---|---|
| Species richness (SR) | Functional diversity (SES.FD) | ||
| Ponds | Management (organic) | 0.32 ± 0.16* | 0.81 ± 0.66 |
| PCoA1 | 0.38 ± 0.34 | 0.52 ± 1.44 | |
| PCoA2 | −0.47 ± 0.62 | −1.83 ± 2.34 | |
| Marginal/Conditional R2 | 0.26/0.26 | 0.10/0.34 | |
| Moran’s I (P-values) | −0.02 (0.91) | −0.04 (0.90) | |
| Landscape features (200 m) | Forest | 0.007 ± 0.003 | 0.18 ± 0.10 |
| Silviculture | 0.004 ± 0.005 | 0.30 ± 0.17 | |
| Marginal/Conditional R2 | 0.13/0.13 | 0.25/0.33 | |
| Moran’s I (P-values) | −0.12 (0.51) | −0.04 (0.68) | |
Non-significant P-values for Moran’s I index indicate a lack of spatial autocorrelation in the model’s residuals.
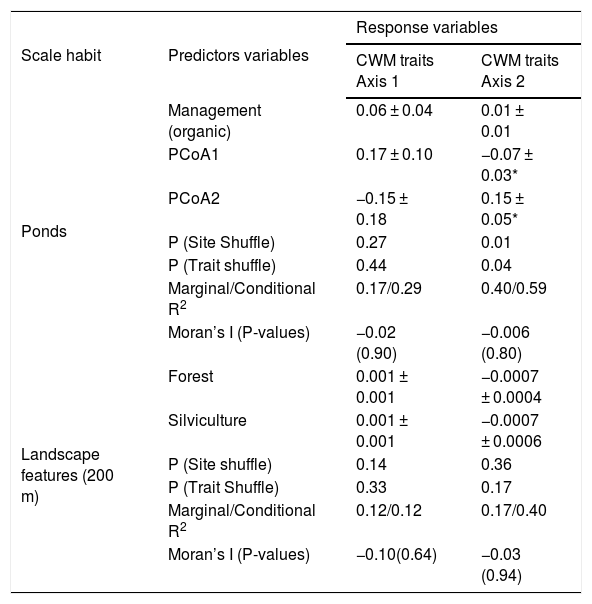
Generalized linear mixed models (GLMMs) relating community-weighted means for traits (axis PCoA species traits) of anurans to management type and environmental conditions, summarized in the first two axes of the principal component coordinates (pond characteristics: PCoA1 and PCoA2) and scale area in farms in southern Brazil.
| Scale habit | Predictors variables | Response variables | |
|---|---|---|---|
| CWM traits Axis 1 | CWM traits Axis 2 | ||
| Ponds | Management (organic) | 0.06 ± 0.04 | 0.01 ± 0.01 |
| PCoA1 | 0.17 ± 0.10 | −0.07 ± 0.03* | |
| PCoA2 | −0.15 ± 0.18 | 0.15 ± 0.05* | |
| P (Site Shuffle) | 0.27 | 0.01 | |
| P (Trait shuffle) | 0.44 | 0.04 | |
| Marginal/Conditional R2 | 0.17/0.29 | 0.40/0.59 | |
| Moran’s I (P-values) | −0.02 (0.90) | −0.006 (0.80) | |
| Landscape features (200 m) | Forest | 0.001 ± 0.001 | −0.0007 ± 0.0004 |
| Silviculture | 0.001 ± 0.001 | −0.0007 ± 0.0006 | |
| P (Site shuffle) | 0.14 | 0.36 | |
| P (Trait Shuffle) | 0.33 | 0.17 | |
| Marginal/Conditional R2 | 0.12/0.12 | 0.17/0.40 | |
| Moran’s I (P-values) | −0.10(0.64) | −0.03 (0.94) | |
Non-significant P-values for Moran’s I index indicate a lack of spatial autocorrelation in the model’s residuals.
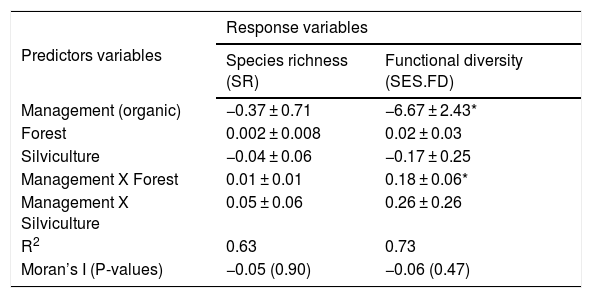
GLM relating species richness and functional diversity (SES.FD) of anurans to management type and landscape features (scale 500 m, forest and silviculture, respectively) in farms in southern Brazil.
| Predictors variables | Response variables | |
|---|---|---|
| Species richness (SR) | Functional diversity (SES.FD) | |
| Management (organic) | −0.37 ± 0.71 | −6.67 ± 2.43* |
| Forest | 0.002 ± 0.008 | 0.02 ± 0.03 |
| Silviculture | −0.04 ± 0.06 | −0.17 ± 0.25 |
| Management X Forest | 0.01 ± 0.01 | 0.18 ± 0.06* |
| Management X Silviculture | 0.05 ± 0.06 | 0.26 ± 0.26 |
| R2 | 0.63 | 0.73 |
| Moran’s I (P-values) | −0.05 (0.90) | −0.06 (0.47) |
Non-significant P-values for Moran’s I index indicate a lack of spatial autocorrelation in the model’s residuals.
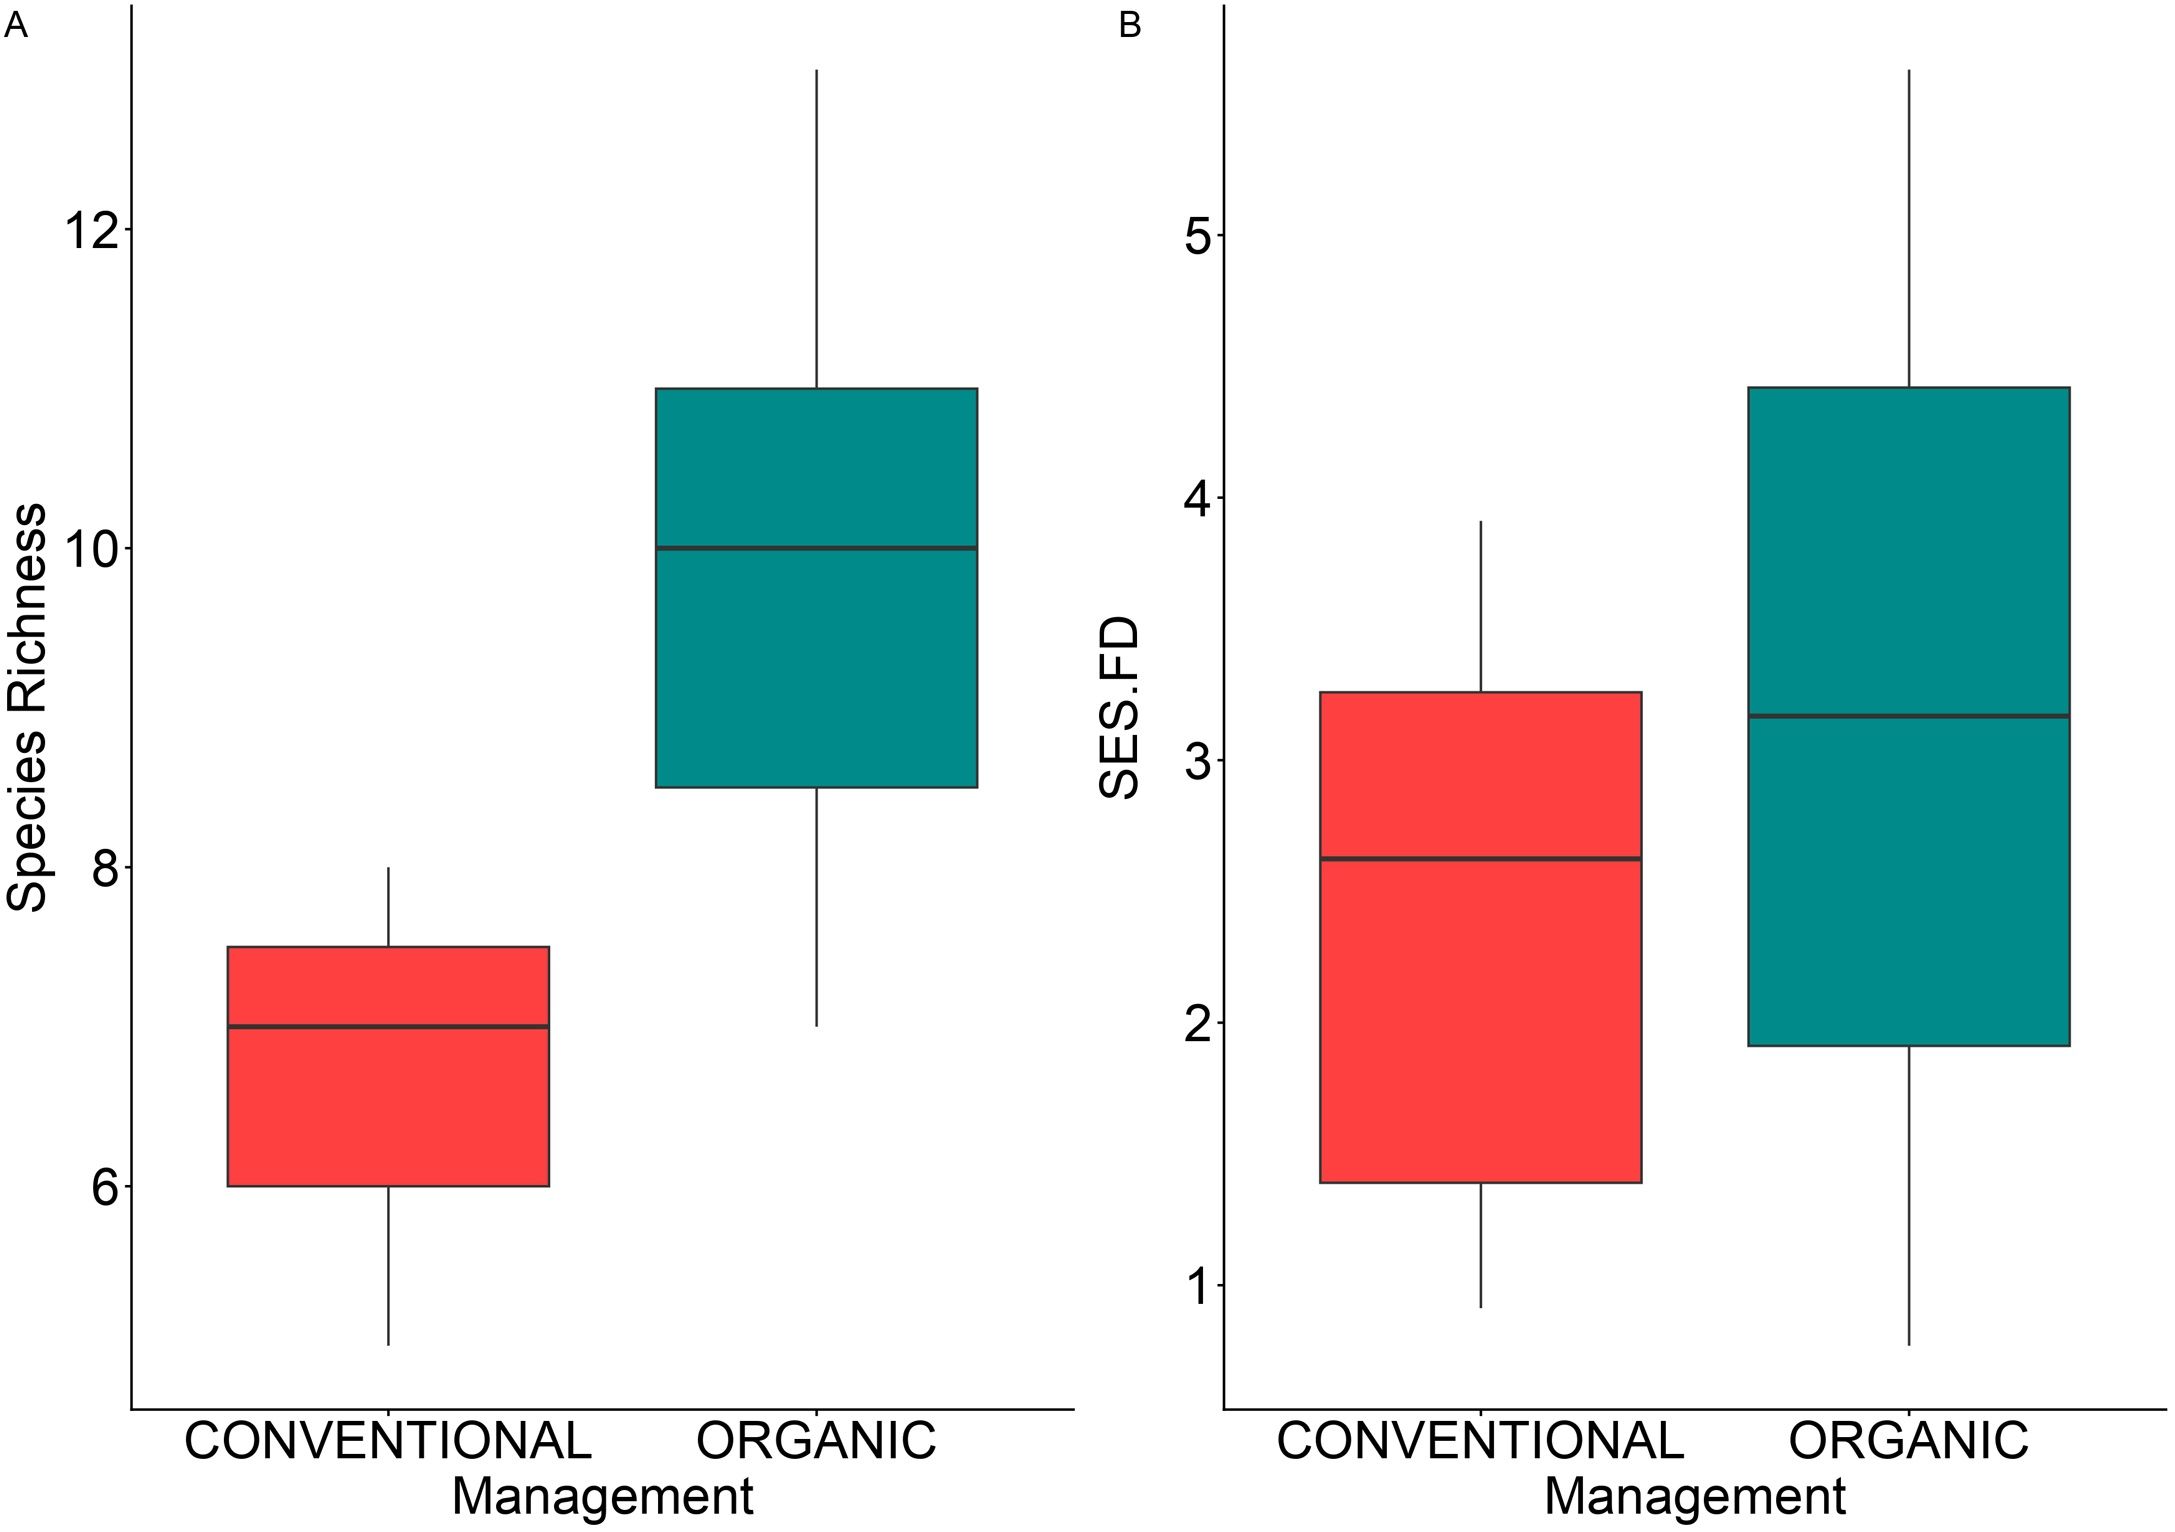
Species richness was higher in organic ponds than in conventional ponds, whereas functional diversity did not differ between agricultural management types on this scale (Table 2; Fig. 1A–B). However, neither metric was related to forest or silviculture cover within 200 m (Table 2).

The anuran species composition differed significantly between ponds from organic and conventional agroecosystems (PERMANOVA, F(1,25) = 2.245, p = 0.017; PERMDISP = F(1,25) = 2.63, p = 0.131). Taxonomic beta diversity was 0.58, driven by turnover (0.38) and nestedness (0.20) (Fig. S2). In contrast, functional composition did not differ significantly (PERMANOVA, F(1,25) = 1.15, p = 0.31; PERMDISP = F(1,25) = 0.16, p = 0.683), with functional beta diversity of 0.70 dominated by nestedness (0.62) (Fig. S3).
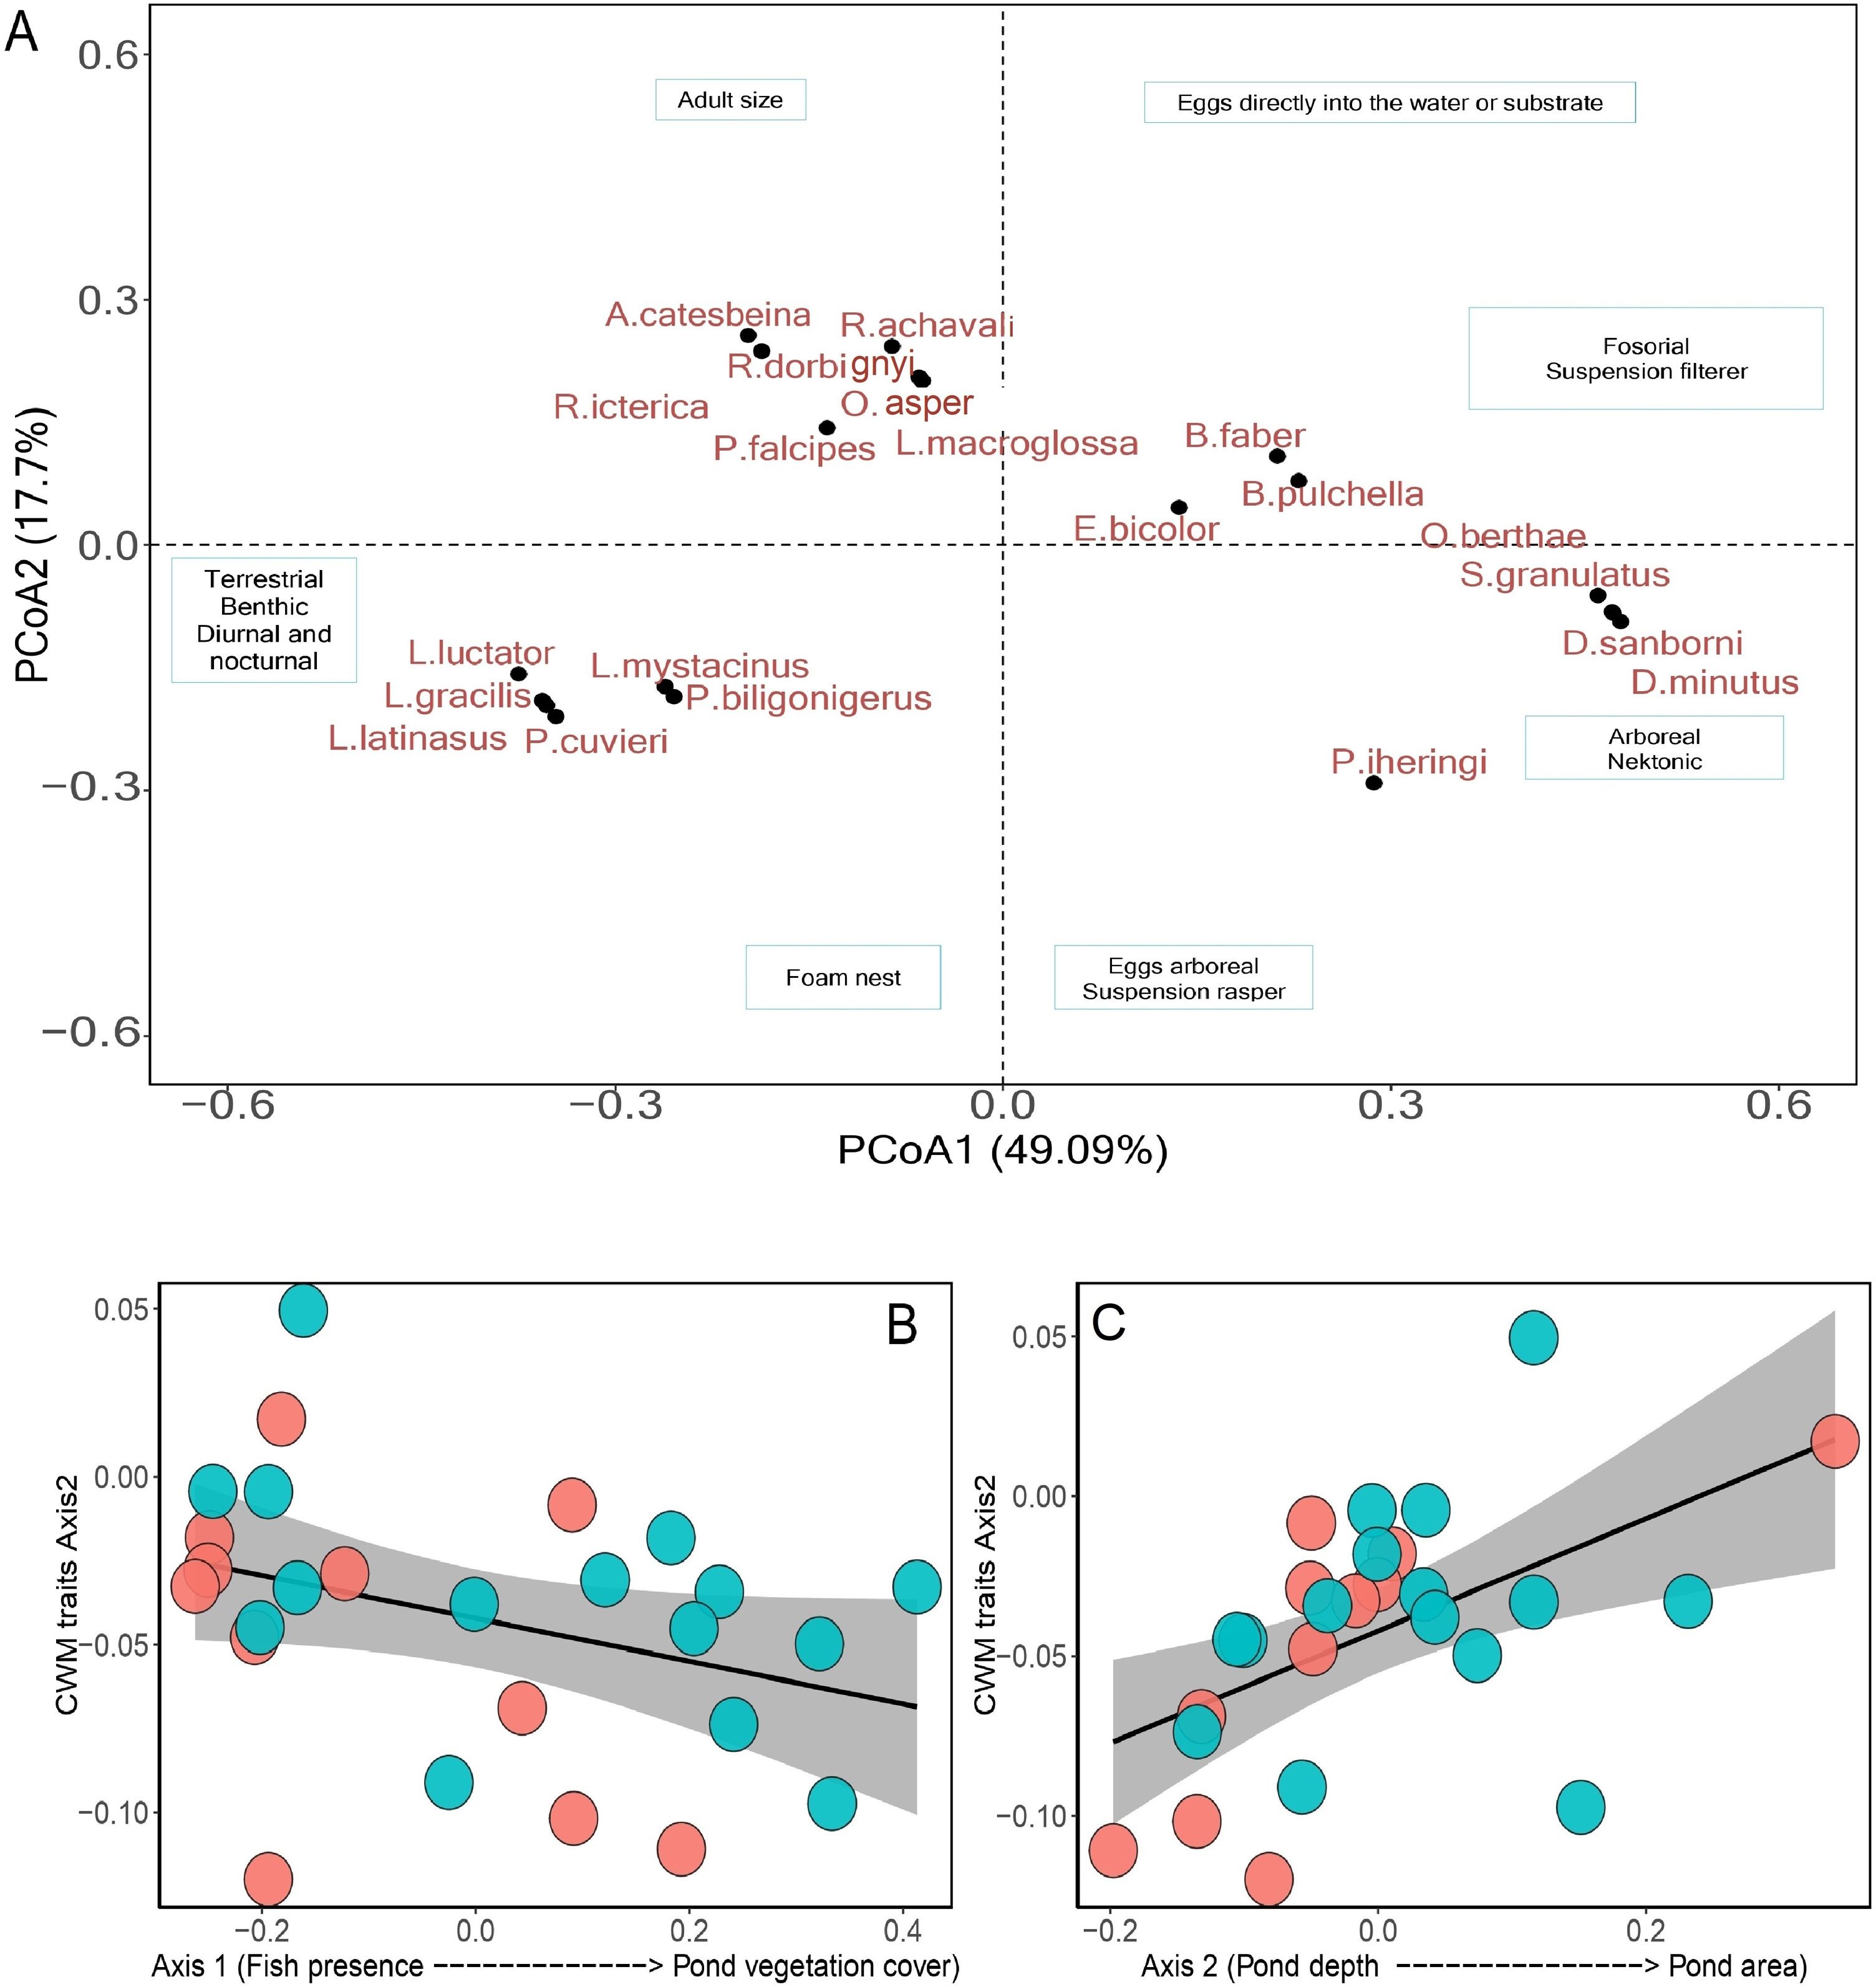
The first two PCoA axes explained 66.79% of trait variation among species (Fig. 2A). Axis 1 represented a gradient from terrestrial species with benthic larvae and mixed activity periods to arboreal or fossorial species with nektonic or suspension-feeding larvae. Neither PCoA1 nor PCoA2 scores were significantly associated with management type, pond characteristics, or landscape variables (Table 3).

The community weighted mean (CWM) traits and their relationship with the characteristic’s ponds (PCoA1 and PCoA2). Only significant trends in CWM are presented here. In section A: PCoA of species traits, B-C: Dots in blue are ponds in organic farming, and red are ponds in conventional farming.
The second PCoA axis was linked to spawning sites and adult body size (SVL), ranging from surface-spawning species to those using foam nests or arboreal eggs (Fig. 2A). While management type had no effect, pond characteristics influenced traits (Table 3): surface-spawning species were less common with greater vegetation cover, which favored foam-nesting or arboreal-egg species (Fig. 2B). Larger ponds supported more surface-spawning species (Fig. 2C). No landscape-scale associations were detected (Table 3).
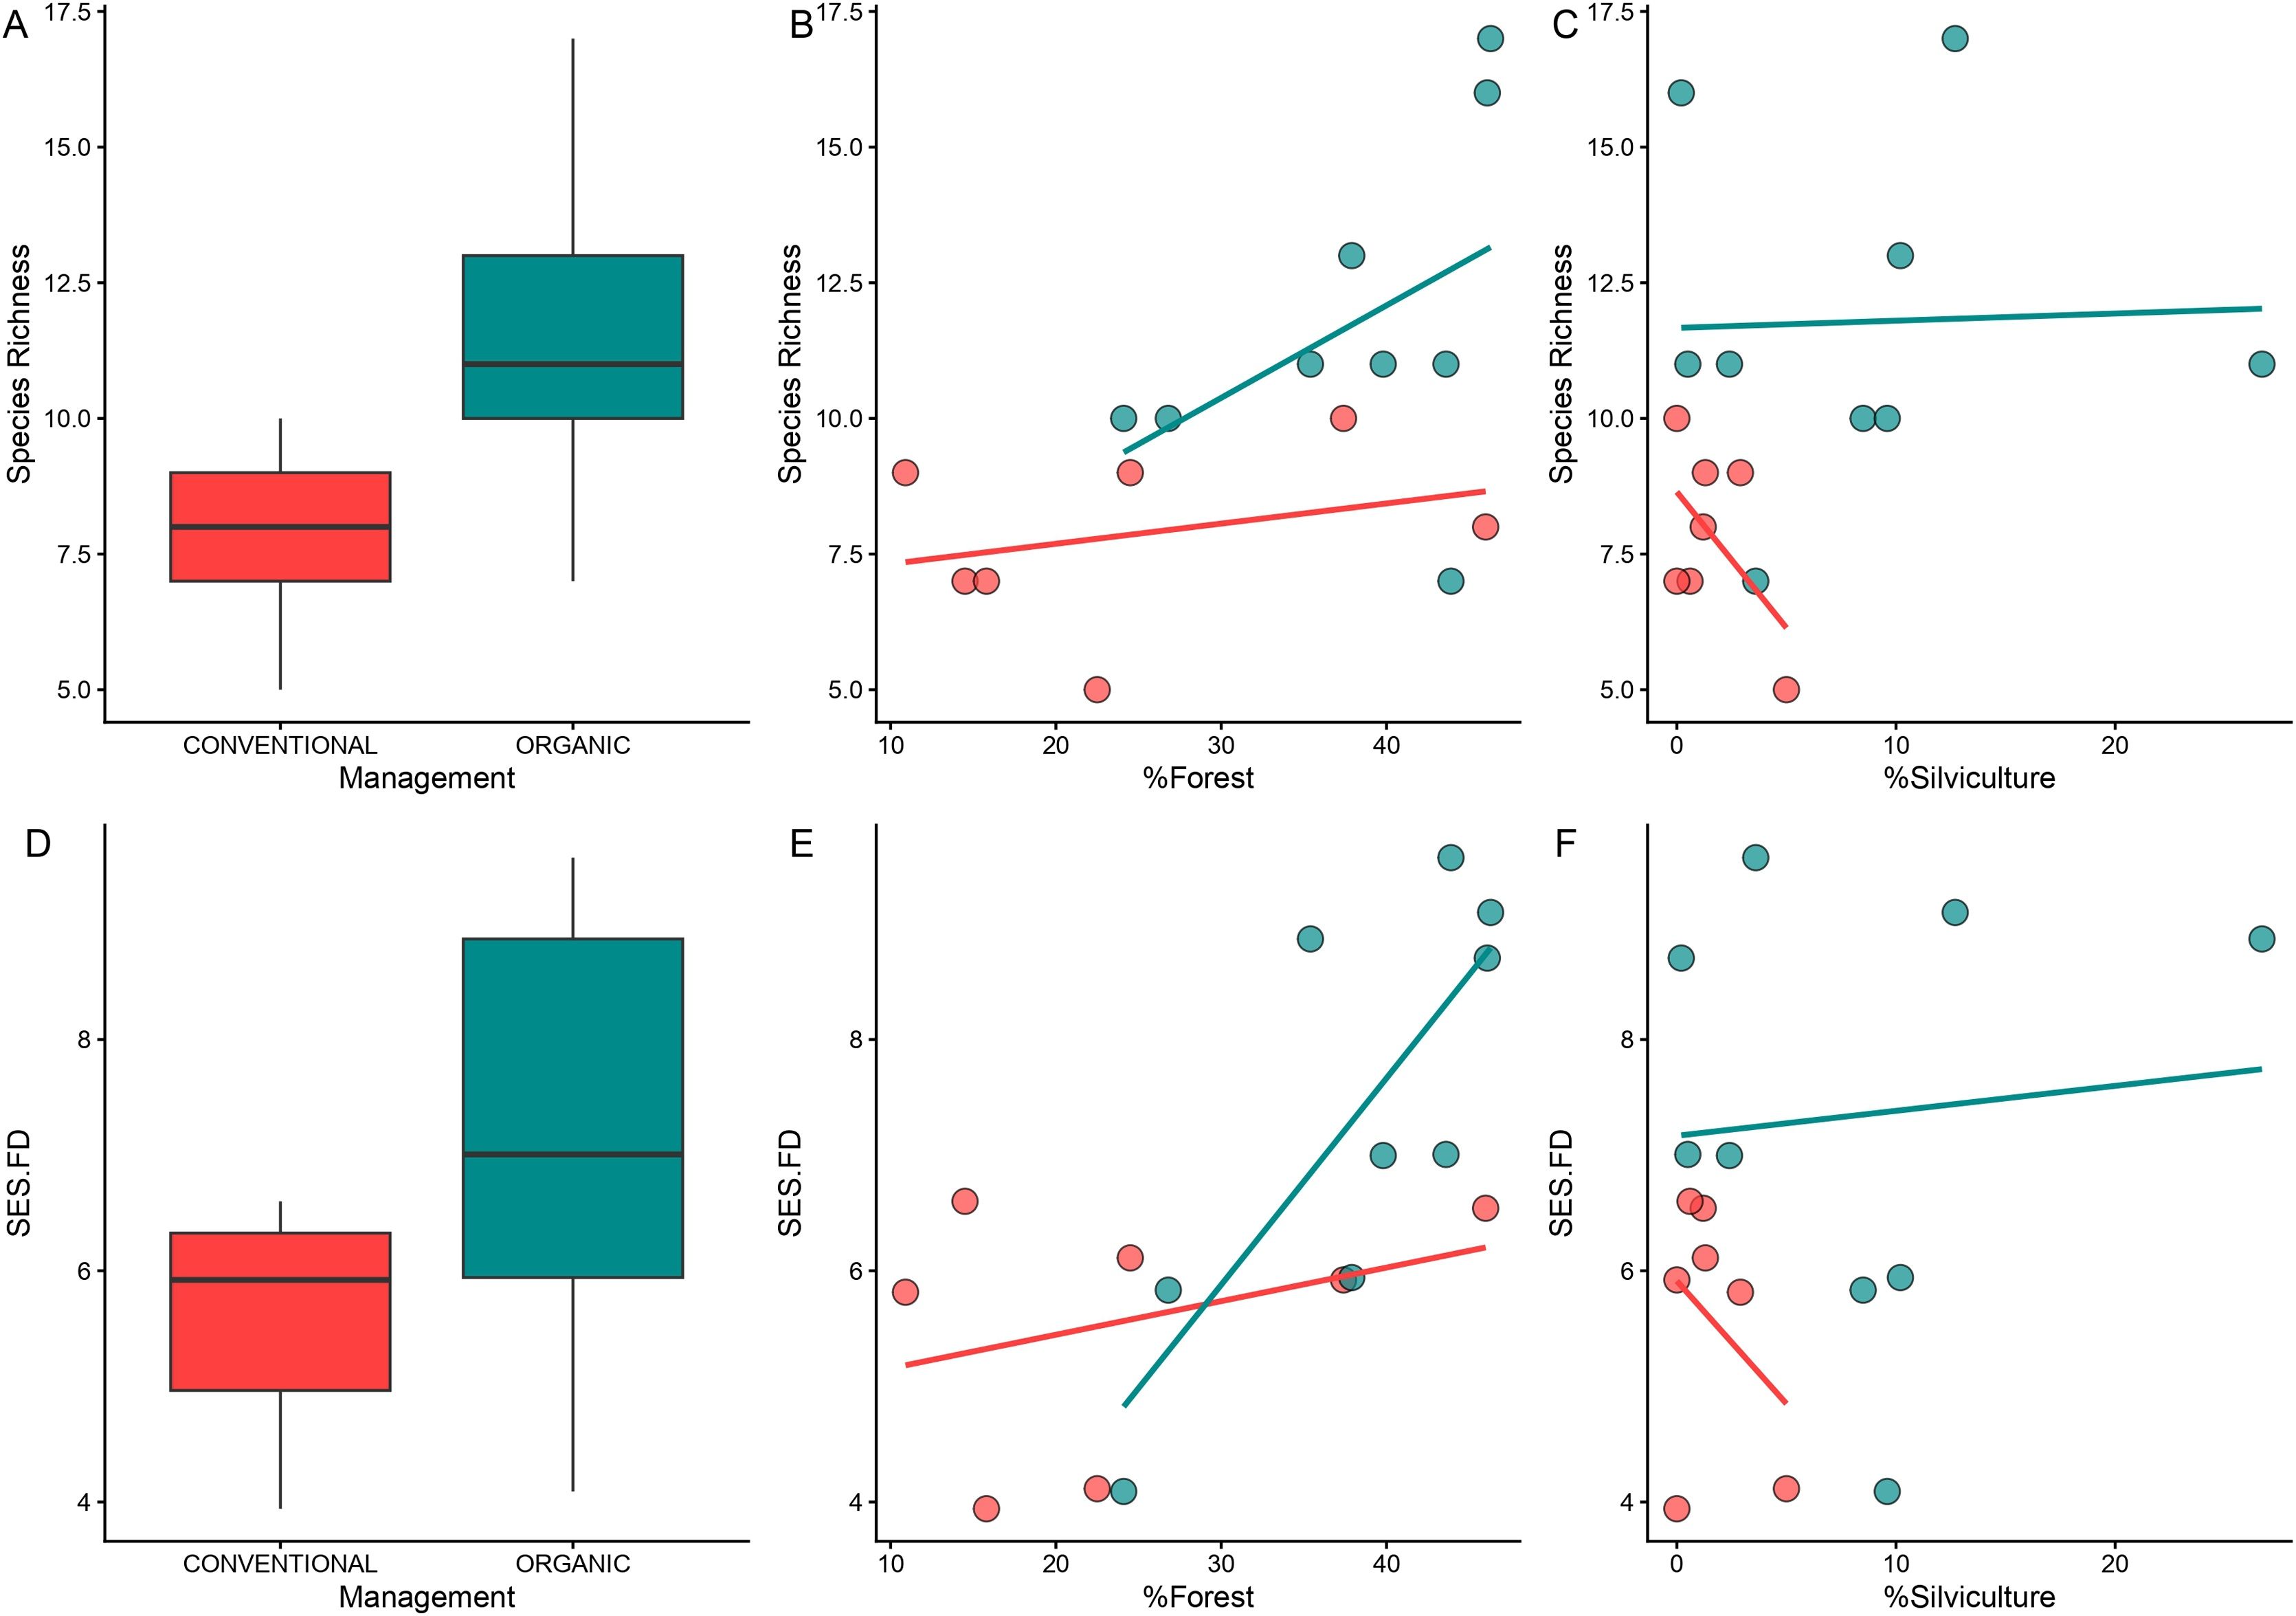
At the farming level, patterns mirrored those at the pond scale: organic farming had higher species richness and functional diversity than conventional ones (Table 4; Fig. 3A–D). The interaction between management and landscape features was not significant for richness (Table 4; Fig. 3B–C), but functional diversity increased with forest cover in organic agroecosystems (Table 4; Fig. 3E–F).

Relationship between the species richness and A: farming management; B-C: interaction between farming management and landscape features (scale 500 m, forest and silviculture, respectively); relationships between functional diversity (SES.FD) and farming management; E-F: interaction between farming management and landscape features (scale 500 m, forest and silviculture, respectively).
Our results demonstrate that anuran diversity patterns in Brazilian Pampa farming are shaped by the combined effects of agricultural management, local habitat characteristics, and landscape context. At the pond scale, species richness was consistently higher in organically managed farming, indicated that organic farming can mitigate biodiversity loss in agricultural landscapes (Tuck et al., 2014; Katayama et al., 2019). These benefits are likely associated with reduced pesticide and lower land-use intensity, which contribute to more favorable conditions for amphibians (Maltchik et al., 2017; Katayama et al., 2019).
In contrast, functional diversity did not differ between management types at the pond scale, indicating that although organic systems support a greater number of species, the range of functional traits represented locally remains similar between organic and conventional ponds. This pattern suggests some degree of functional similarity among anuran species occupying agricultural ponds, whereby species turnover does not necessarily translate into changes in functional diversity (Pereyra et al., 2018). Similar decoupling between taxonomic and functional diversity has been reported in amphibian assemblages exposed to agricultural intensification (Pereyra et al., 2018).
Despite this functional similarity at the local scale, taxonomic composition differed significantly between ponds in organic and conventional farming. Species replacement rather than nested species loss dominated taxonomic beta diversity, indicating that management practices filter species identities without eliminating functional strategies. Conventional farming was likely dominated by disturbance-tolerant and generalist species, while organically managed systems supported a broader set of species (Flynn et al., 2009; Agostini et al., 2021). This taxonomic turnover without corresponding functional divergence highlights the importance of considering multiple dimensions of biodiversity when assessing the ecological effects of agricultural practices (Pereyra et al., 2018.
Analyses of community-weighted mean traits further revealed that functional trait composition was more strongly associated with breeding site characteristics than with management type. Pond vegetation cover and pond size influenced the distribution of reproductive strategies and body size, favoring species that use foam nests or arboreal egg deposition in structurally complex habitats. For instance, species such as Phyllomedusa iheringii and foam-nesting Leptodactylidae were favored by structurally complex ponds, whereas open, simplified ponds tended to support more generalist taxa (Moreira et al., 2020). Vegetation plays a critical role during amphibian reproduction by providing oviposition sites, shelter, and foraging habitat for larvae, while also reducing exposure to agrochemicals (Agostini et al., 2021). The loss of aquatic vegetation, often associated with herbicide use in agricultural systems, can therefore negatively affect amphibian reproductive success and survival (Agostini et al., 2020).
At broader spatial scales, landscape context emerged as a key driver of functional diversity. While landscape composition within 200 m of ponds was not associated with diversity metrics, functional diversity at the farming level increased with forest cover in organic systems. This scale-dependent response suggests that local breeding habitats alone are insufficient to maintain functional diversity and that access to surrounding natural habitats is critical for sustaining a wider range of ecological strategies (Ribeiro et al., 2017; Moreira et al., 2020). Forest patches likely function as refuges and sources for recolonization, enhancing functional complementarity in organically managed landscapes (Ribeiro et al., 2017).
The contrasting effects of forest cover and silviculture further emphasize the importance of landscape quality. Monoculture plantations, such as eucalyptus plantations common in this region, can reduce habitat suitability and connectivity for amphibians, particularly when combined with intensive management practices (Saccol et al., 2017). In contrast, landscapes that integrate organic farming with native vegetation may better support functionally diverse assemblages.
Overall, our findings indicate that organic farming in the Brazilian Pampa support higher anuran species richness and, at broader spatial scales, greater functional diversity when embedded within landscapes containing native forest cover. These results underscore the importance of integrating sustainable agricultural practices with landscape-level conservation strategies to mitigate biodiversity loss and maintain ecosystem functioning in grassland agroecosystems (Agostini et al., 2021). Policies that promote organic farming alongside the conservation and restoration of natural habitats may therefore play a crucial role in reconciling agricultural production with biodiversity conservation.
FundingCJCP thanks CAPESfor a master's scholarship. This research was funded by FAPERGS (proc.21/2551-0001950-6), andCNPq (proc.406414/2021-1). LD research has been funded by a CNPq Productivity Fellowship (grant 306951/2022-3).
The authors declare that they have no known competing financial interests or personal relationships that could have appeared to influence the work reported in this paper.
We thank the farm owners for allowing us access to their properties to conduct this study. We also thank Camila Medeiros, Orlando Hernandez, and Gabriel Dubal for their assistance during the fieldwork. To Fernando Becker for his help in the landscape analysis. To Jose Tovar Marquez, thank you for the comments made on the initial version of this manuscript. This work is a contribution of the National Institute of Science and Technology (INCT) in Ecology, Evolution, and Biodiversity Conservation funded by CNPq (grants 465610/2014-5 and409197/2024-6) and FAPEG (grant201810267000023).
The following are Supplementary data to this article: