




Despite their ecological importance, carnivorans are often underrepresented in protected areas (PAs), making it crucial to evaluate the representation of their richness and endemicity patterns within these areas for effective conservation. The Yucatan Peninsula (YP), a unique biogeographic province, harbors 18 carnivoran species (∼22% of the Americas’ carnivoran diversity). Using ecological niche modeling and diversity range analysis, we assessed the spatial representation of these patterns within the region’s PAs. Our results show that peak species richness occurs in southern Quintana Roo, southeastern Campeche, the Tabasco-Chiapas border (Mexico), and northern Belize-Guatemala, while endemicity is highest on Cozumel Island and in south-central Tabasco. However, only 9.48 % of high-richness and high-endemicity areas lie within existing PAs. Key PAs partially covering these priority zones include Sierra del Lacandón, Laguna del Tigre, Tikal, and Yaxhá-Nakum-Naranjo National Parks (Guatemala); the Rio Bravo Conservation Area (Belize); and the Calakmul Biosphere Reserve (Mexico). These findings underscore the need to expand PA coverage and enhance systematic assessments of biodiversity patterns within them to safeguard the YP’s unique carnivoran assemblages and their ecosystem functions.

Carnivorans play a critical role in maintaining ecosystem balance, influencing nutrient distribution, and regulating prey populations (Schmitz et al., 2010; Estes et al., 2011). Their presence often has cascading effects on biodiversity and ecological processes, making them essential to the health of entire ecosystems. Consequently, their conservation is essential not only for preserving ecological interactions but also for maintaining the integrity and structure of communities (Ripple et al., 2014; Camargo-Sanabria et al., 2015; Wolf and Ripple, 2017). Due to their charismatic nature and role as umbrella species, carnivorans are particularly useful for conservation planning, as their protection often benefits numerous other species within their geographic range (Steenweg et al., 2023). However, carnivoran populations are currently declining due to habitat loss and degradation, reduced prey availability, illegal wildlife trade, and human-wildlife conflicts in urban, agricultural, and livestock areas (Ripple et al., 2014; Wolf and Ripple, 2017; Asociación Mexicana de Mastozoología and Word Wildlife Fund, 2022). These threats are part of a larger global biodiversity crisis, with Earth facing its greatest environmental challenge in recent history. Extinction rates are currently hundreds or even thousands of times higher than those observed in the past ten million years, largely due to human activities (Díaz et al., 2019; Ceballos et al., 2020).
Protected Areas (PAs) are a cornerstone of global conservation strategies, helping to mitigate anthropogenic threats and safeguarding species the effects of climate change among other threats (Hannah et al., 2007; Pérez Juárez et al., 2023). PAs promote in situ conservation, which is one of the most effective approaches for preserving biodiversity, ecosystem integrity, and environmental services (García-Frapolli et al., 2009). Furthermore, PAs contribute significantly to scientific research, education, and local economies through activities such as ecotourism and sustainable forestry. They also hold cultural and heritage value for local and Indigenous communities (García-Frapolli et al., 2009). However, the establishment of PAs has often been influenced by economic interests, leading to their placement in residual zones that do not conflict with economic development, rather than in areas of high conservation value (Devillers et al., 2015; Terraube et al., 2020). This has resulted in significant challenges related to the representativeness and efficiency of PAs (Vieira et al., 2019). Latin America is no exception to this trend, and its PAs often suffer from suboptimal placement, which undermines their effectiveness (e.g., Figueroa and Sánchez-Cordero, 2008; Sims and Alix-Garcia, 2017). Therefore, identifying sites with high species richness and endemicity is crucial for improving the representativeness of PAs (Soberón et al., 2021).
The Yucatan Peninsula (YP), spanning parts of Mexico, Belize, and Guatemala, serves as an important case study for carnivoran conservation. Recognized as a unique biogeographical province, it hosts exceptional biodiversity, including 18 carnivoran species—about 22% of all carnivorans in the Americas (Islebe et al., 2015; Reyna-Hurtado et al., 2015; Durán-García et al., 2016). Among these are threatened species like the jaguar (Panthera onca Linnaeus, 1758) and the critically endangered Cozumel raccoon (Procyon pygmaeus Merriam, 1901), an endemic found only on Cozumel Island (Asociación Mexicana de Mastozoología and Word Wildlife Fund, 2022; Cuarón et al., 2004). The YP’s dense forests, the second-largest in the Americas after the Amazon, provide critical habitat for these species (Durán-García et al., 2016). Yet, like many regions, the YP faces challenges in PA representativeness, with conservation gaps that are currently widening due to the boom in mass tourism—a trend that may leave key species unprotected (Figueroa and Sánchez-Cordero, 2008).
This study examines carnivoran diversity patterns within and outside PAs, using the YP as a model system to explore broader conservation strategies. By analyzing species richness and endemicity through ecological niche models (ENMs) and diversity range analyses (Soberón et al., 2021), we identify high-priority zones for carnivoran conservation. Our findings can guide PA expansion, wildlife management policies, and mitigation strategies to enhance species resilience against anthropogenic pressures. Given carnivorans’ role as umbrella species, protecting them benefits entire ecosystems, making this research relevant not only to the YP but to global biodiversity conservation efforts.
MethodsTo study species richness and endemicity patterns and their representation in the PAs of the YP, we conducted a diversity-range analysis. This quantitative method identifies areas of high species richness and endemicity (defined by low dispersion field values, Borregaard and Rahbek, 2010) and assesses their statistical significance by comparing observed patterns with null distributions generated through randomization of presence-absence matrices (PAMs), a fundamental unit of analysis in community ecology (Götzenberger et al., 2012). The core of this analysis is the dispersion field metric. Originally conceptualized by Smith (1983) and Graves and Rahbek (2005), it is defined for a given locality as the mean geographic range size of all species present there. As demonstrated by Soberón and Ceballos (2011), this measure is mathematically equivalent to the mean number of species a focal site shares with all other sites in the study area. Consequently, the dispersion field serves as an inverse metric of endemicity. A low value indicates that a site hosts species with very restricted distributions (few shared species with other sites), characteristic of high endemicity. Conversely, a high value reflects a community dominated by widespread species (many shared species). Below, we describe the methods used to estimate potential species distributions, construct PAM, and perform the diversity-range analysis.
Potential distribution modelingData collection and preparationWe defined our study area based on the Yucatan Platform (French and Schenk, 2004) extended by a 100 km buffer. This distance was selected to account for two key factors: (1) the potential dispersal capacity of the largest target species (e.g., Puma concolor Linnaeus 1771; González-Borrajo et al., 2017), and (2) the scale of regional environmental gradients relevant to the species distribution. We compiled a list of carnivoran species present in the region through a literature review and scientific collection databases. Based on this list, species occurrence data were obtained from open primary biodiversity data, including the Global Biodiversity Information Facility (GBIF, https://www.gbif.org/; GBIF, 2025), VerNet (http://vertnet.org/), the Arctos Database (https://arctos.database.museum/), the Sistema Nacional de Información Sobre Biodiversidad (SNIB, https://www.snib.mx/), and iNaturalist (https://www.inaturalist.org/). Additional records were sourced from published studies (e.g., Nagy-Reis et al., 2020). Data cleaning followed standard protocols for primary diversity records (Cobos et al., 2018): we removed fossil records, incorrectly georeferenced localities, duplicate entries, and dubious occurrences. To ensure better correspondence with environmental data, records predating 1990 were excluded (Tuanmu and Jetz, 2014; Venter et al., 2016). Spatial autocorrelation was addressed by thinning occurrence records to a minimum distance of 5 km using the R package ntbox (Osorio-Olvera et al., 2020a). After a curation process starting from 774,917 initial occurrences, we retained 140,068. This final dataset was then split into training (70%) and testing (30%) subsets.
Environmental dataAs a predictor of distribution, we used WorldClim 2 data (Fick and Hijmans, 2017), which provide interpolated climate and precipitation averages for the period 1970–2000. Additionally, we incorporated SoilTemp variables (Lembrechts et al., 2020), which offer ground-level temperature data reflecting microclimatic conditions that influence vegetation and species distributions (Haesen et al., 2021; Lembrechts et al., 2022). Other variables included tree cover (Tuanmu and Jetz, 2014) and human footprint (Venter et al., 2016), both of which have been shown to significantly affect species distributions (Basille et al., 2009; Parsons et al., 2018; Contreras-Díaz et al., 2022; Sánchez-Reyes et al., 2023). All raster layers were obtained at a spatial resolution of ∼1 km².
To reduce multicollinearity-related issues in the niche models, we calculated Spearman correlations between environmental variables associated with species occurrences and retained only those with correlation coefficients ≤ 0.7. WorldClim 2 variables 8, 9, 18, and 19 were excluded due to abrupt discontinuities, which are considered artifacts in some regions (Anderson and Raza, 2010; Escobar et al., 2014; Alkishe et al., 2022).
Species distribution modelingWe estimated potential distributions using minimum volume ellipsoids (MVEs, Van Aelst and Rousseeuw, 2009; Qiao et al., 2016), a method chosen for several reasons: i) theoretical and empirical studies have shown that ellipsoid centroid distance correlates with fitness attributes such as population abundance and genetic diversity (Jiménez et al., 2019; Ochoa-Zavala et al., 2022; Osorio-Olvera et al., 2019, 2020b); ii) its convex shape aligns with fundamental niche concepts (Jiménez and Soberón, 2022); iii) MVEs require only three parameters (centroid, number of calibration points, and covariance matrix), minimizing assumptions and computational complexity; iv) MVEs have similar performance to more complex algorithms like MaxEnt (Osorio-Olvera et al., 2020b; Nava-Bolaños et al., 2022).
MVE models were constructed by calibrating different algorithms within a species-specific area to estimate the species' environmental preferences and delimit its geographic distribution (Rojas-Soto et al., 2024). These calibration areas were defined by creating buffer zones around occurrence records, accounting for dispersal limitations and biogeographic barriers (Soberón and Peterson, 2005; Barve et al., 2011). Using the ntbox R package (Osorio-Olvera et al., 2020a), we extracted environmental background data from the calibration areas. Although MVE is a presence-only algorithm, ntbox uses the background data to estimate key metrics for evaluating model performance and significance, including: (1) the proportion of background points within the niche which gives an estimation of how big is the niche relative to the calibration area, (2) the AUC of the ROC curve, (3) the partial ROC test (Peterson et al., 2008), and (4) the binomial test (Osorio-Olvera et al., 2020a,b). We applied the ellipsoid_selection function from the ntbox package to calibrate ellipsoids in 3, 4, 5, and 6 dimensions using all combinations of non-correlated environmental variables. The best model for each species was selected based on three criteria: (a) statistical significance in partial ROC tests (P < 0.05, Peterson et al., 2008), (b) low omission rates for training and testing data (≤0.05%), and (c) higher AUC values. Finally, the best model for each species was binarized using the tenth percentile threshold of the training data.
Diversity range analysisUsing the models2pam function from the bamm R package (Soberón and Osorio-Olvera, 2023; Osorio-Olvera et al., 2024), we constructed a presence-absence matrix (PAM) based on binarized species distribution models. A PAM is defined as an N sites × S species binary matrix, where a value of 1 indicates the presence of species j in cell i, and 0 indicates its absence. This matrix served as the main input for the diversity-range analysis, a robust statistical method that leverages biodiversity presence-absence data to comprehensively describe community composition in terms of species richness and levels of endemicity across a defined study area (Arita et al., 2008; Borregaard and Rahbek, 2010; Soberón et al., 2021; Soberón and Cavner, 2015; Soberón and Ceballos, 2011). A key component of this analysis is the calculation of dispersion fields. For a given cell, its value represents the mean range size of all species occupying it. Dispersion fields serve as an inverse measure of endemicity, with smaller values indicating higher levels of endemicity (Soberón et al., 2021). To assess the statistical significance of the dispersion field values, we randomized the PAM 10,000 times using the diversity_range_analysis function in the bamm package (Osorio-Olvera et al., 2024). Observed dispersion field values were compared to null distributions, with significance thresholds set at 2.5% (lower limit) and 97.5% (upper limit). Cells with dispersion field values below the lower limit were classified as high-endemicity sites, while those above the upper limit were classified as low-endemicity sites. Species richness, on the other hand, is the sum of all the species present in a given cell. Its values are interpreted as follows: low significant values (below the 25th percentile) indicate low richness, high values (above the 75th percentile) indicate high richness, and intermediate richness corresponds to values between the 25th and 75th percentiles (Soberón et al., 2021).
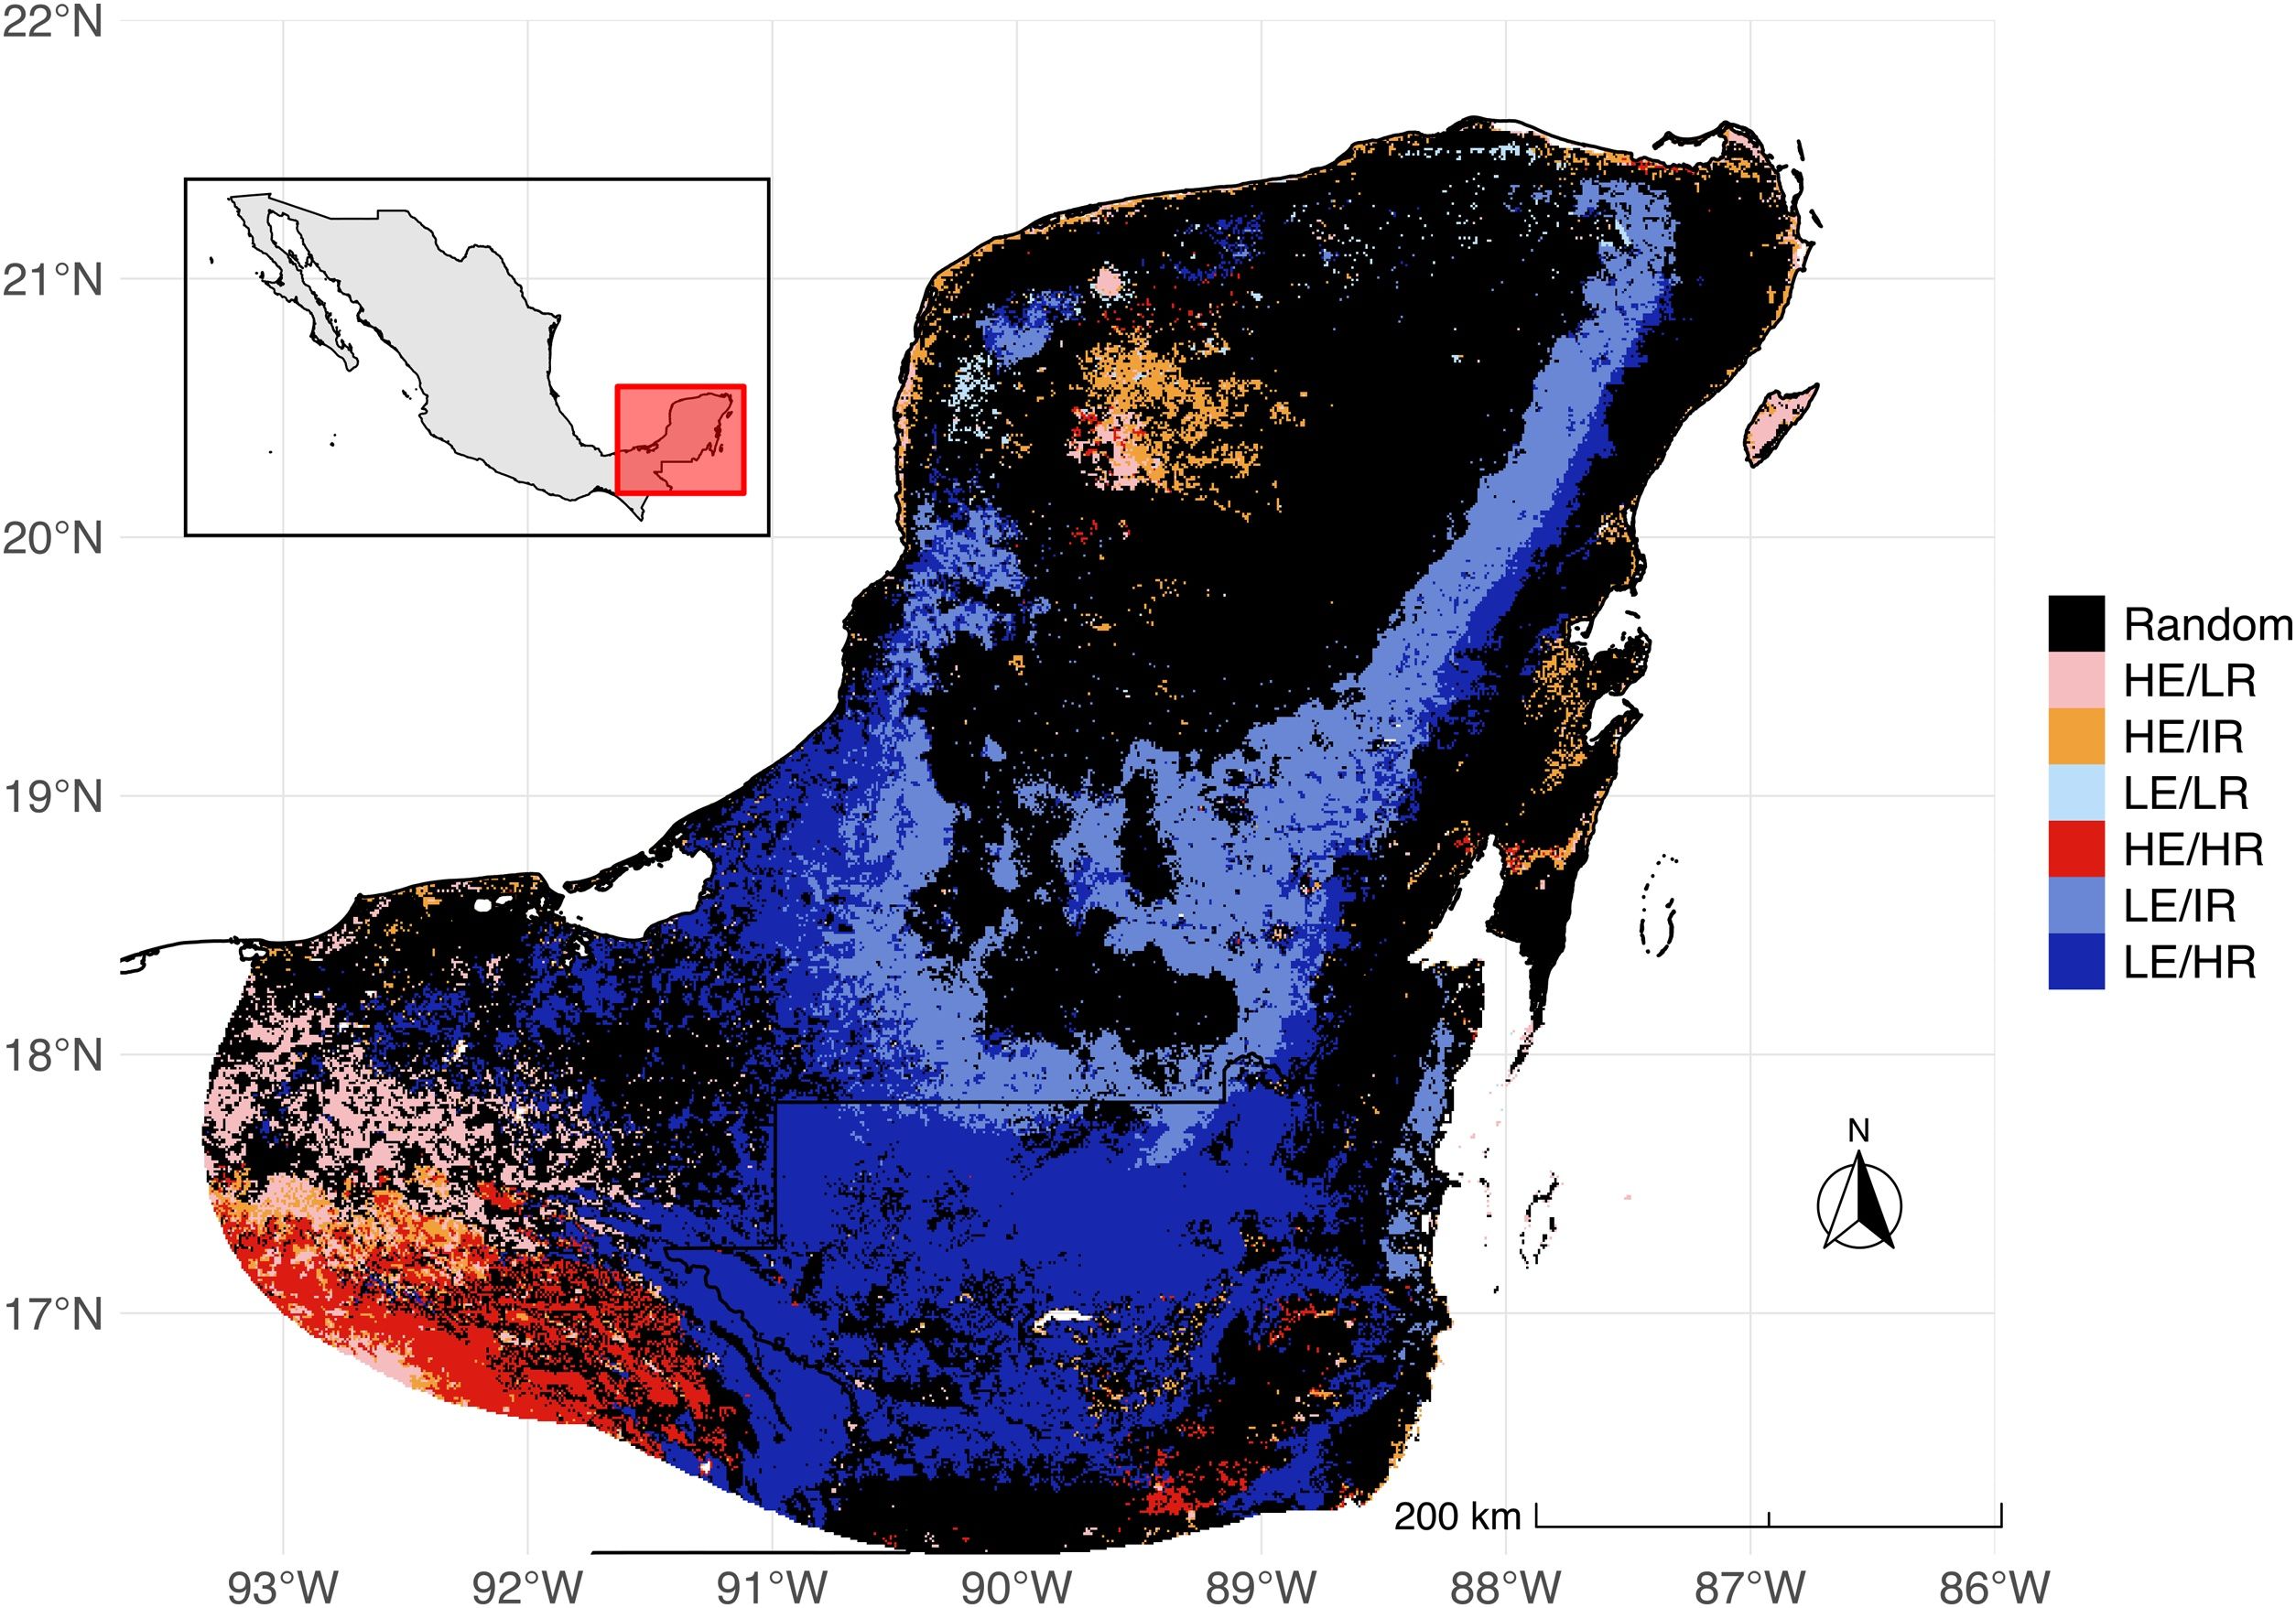
The diversity-range analysis classifies the study area into seven categories based on endemicity and species richness: i) low endemicity and low richness (LE/LR), ii) high endemicity and low richness (HE/LR), iii) low endemicity and intermediate richness (LE/IR), iv) high endemicity and intermediate richness (HE/IR), v) low endemicity and high richness (LE/HR), vi) high endemicity and high richness (HE/HR), and vii) a random pattern (Random), where values of richness and endemicity cannot be distinguished from null distributions. The analysis produced three maps: one for species richness, one for dispersion fields, and one for biodiversity ranges. The last map is a combination of the first two and provides a detailed spatial representation of biodiversity patterns across the study region. These outputs are critical for identifying priority conservation areas and informing strategies to protect species richness and endemicity in the face of anthropogenic pressures.
Protected areasWe obtained PA polygons from Protected Planet: The World Database on Protected Areas (WDPA) and World Database on Other Effective Area-based Conservation Measures 2024, the most comprehensive global databases for marine and terrestrial PAs. We retained PAs with the status of "designated", "registered", or "established", discarding those that had the status of "adopted", "not reported" or "proposed". Only PAs with detailed geographic information and IUCN conservation categories I–VI, which indicate effective management and conservation, were included.
To visualize the distribution of these categories within the most significant PAs, we created a map displaying the percentages of the seven endemicity and species richness categories for the largest PAs. Specifically, we retained only the top 20% of PAs based on area, ensuring that the analysis focused on the most extensive and potentially impactful conservation areas. This approach allowed us to identify how well the largest PAs in the YP represent regions of high biodiversity and endemicity, providing critical insights for prioritizing conservation efforts and enhancing the effectiveness of the PA network.
ResultsA total of 18 carnivoran species were recorded for the Yucatan Peninsula (YP), representing 16 genera and five families (see supplementary material). According to the IUCN Red List of Threatened Species, 14 species are categorized as Least Concern, three as Near Threatened, and one, Procyon pygmaeus, as Critically Endangered. Regarding international trade regulations, five species are listed in CITES Appendix I, two in Appendix II, and two in Appendix III (https://cites.org/eng/app/appendices.php).
During the model selection process, we evaluated between 42 and 6370 models per species, resulting in a total of 38,724 models. Of these, between 16 and 5167 models met the selection criteria. For subsequent analyses, only the best-ranked model for each species was retained. The most frequently selected variables in the best models were annual mean temperature (bio1), isothermality (bio3), and tree cover.
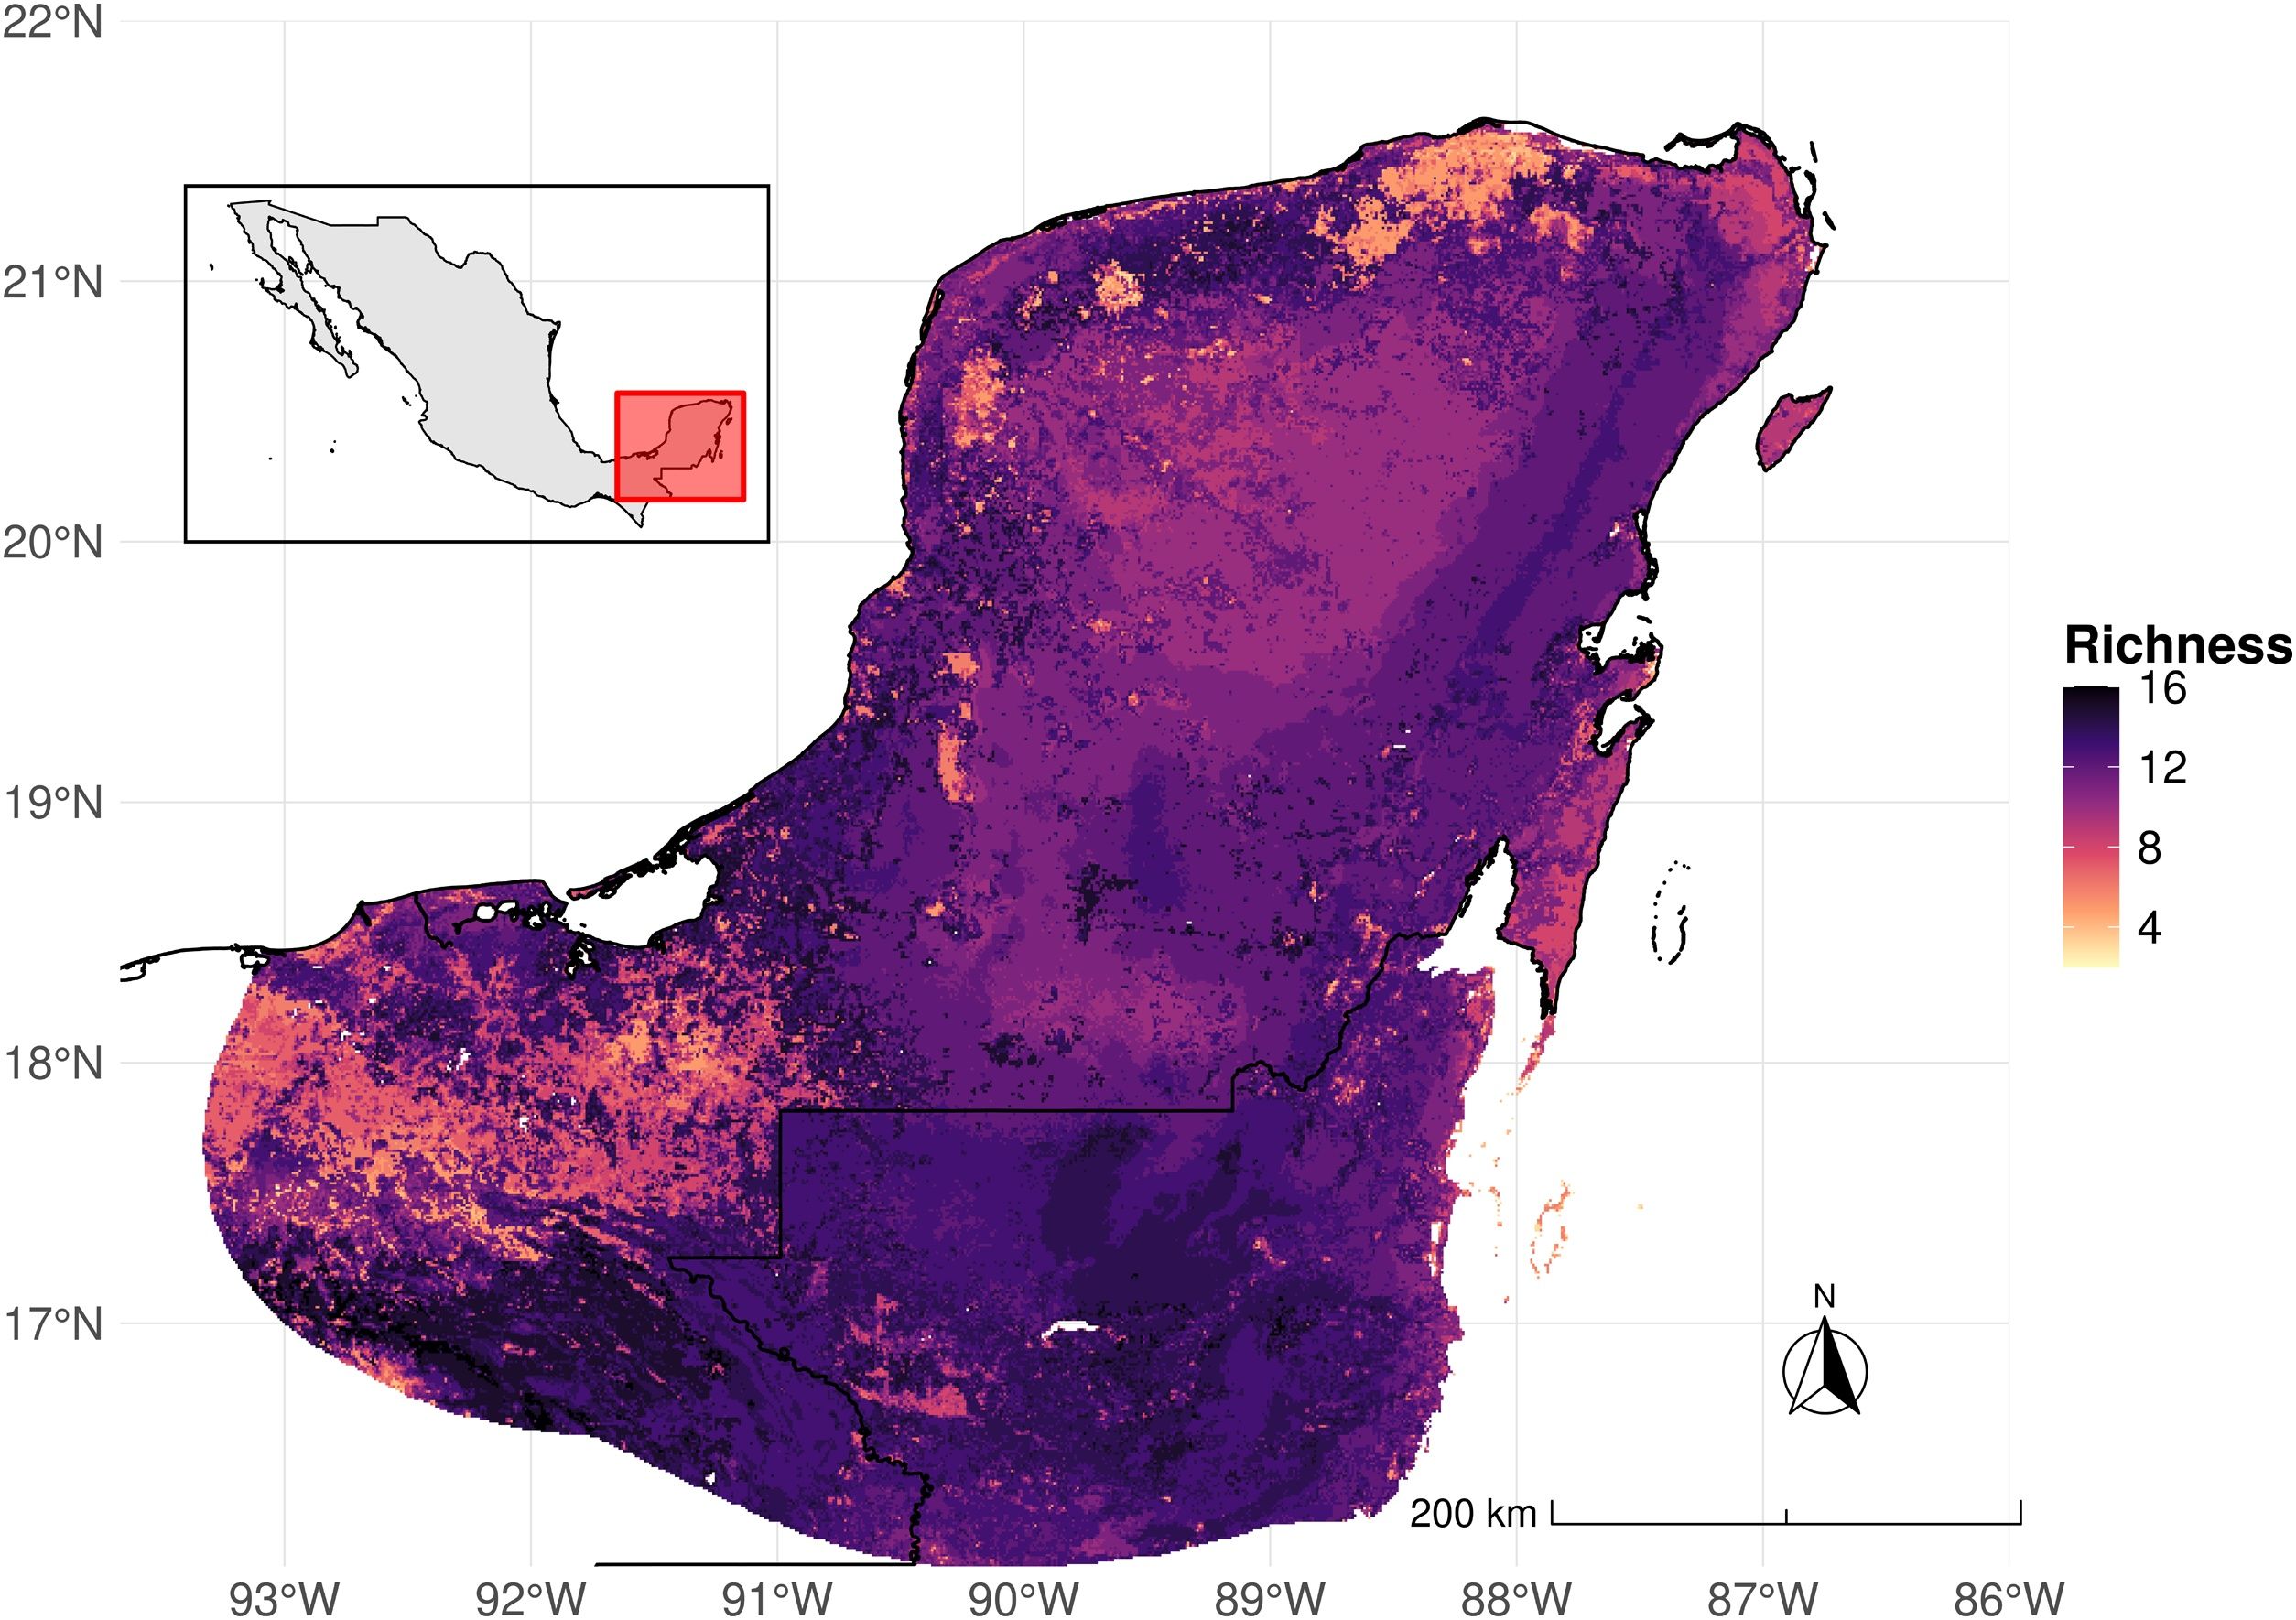
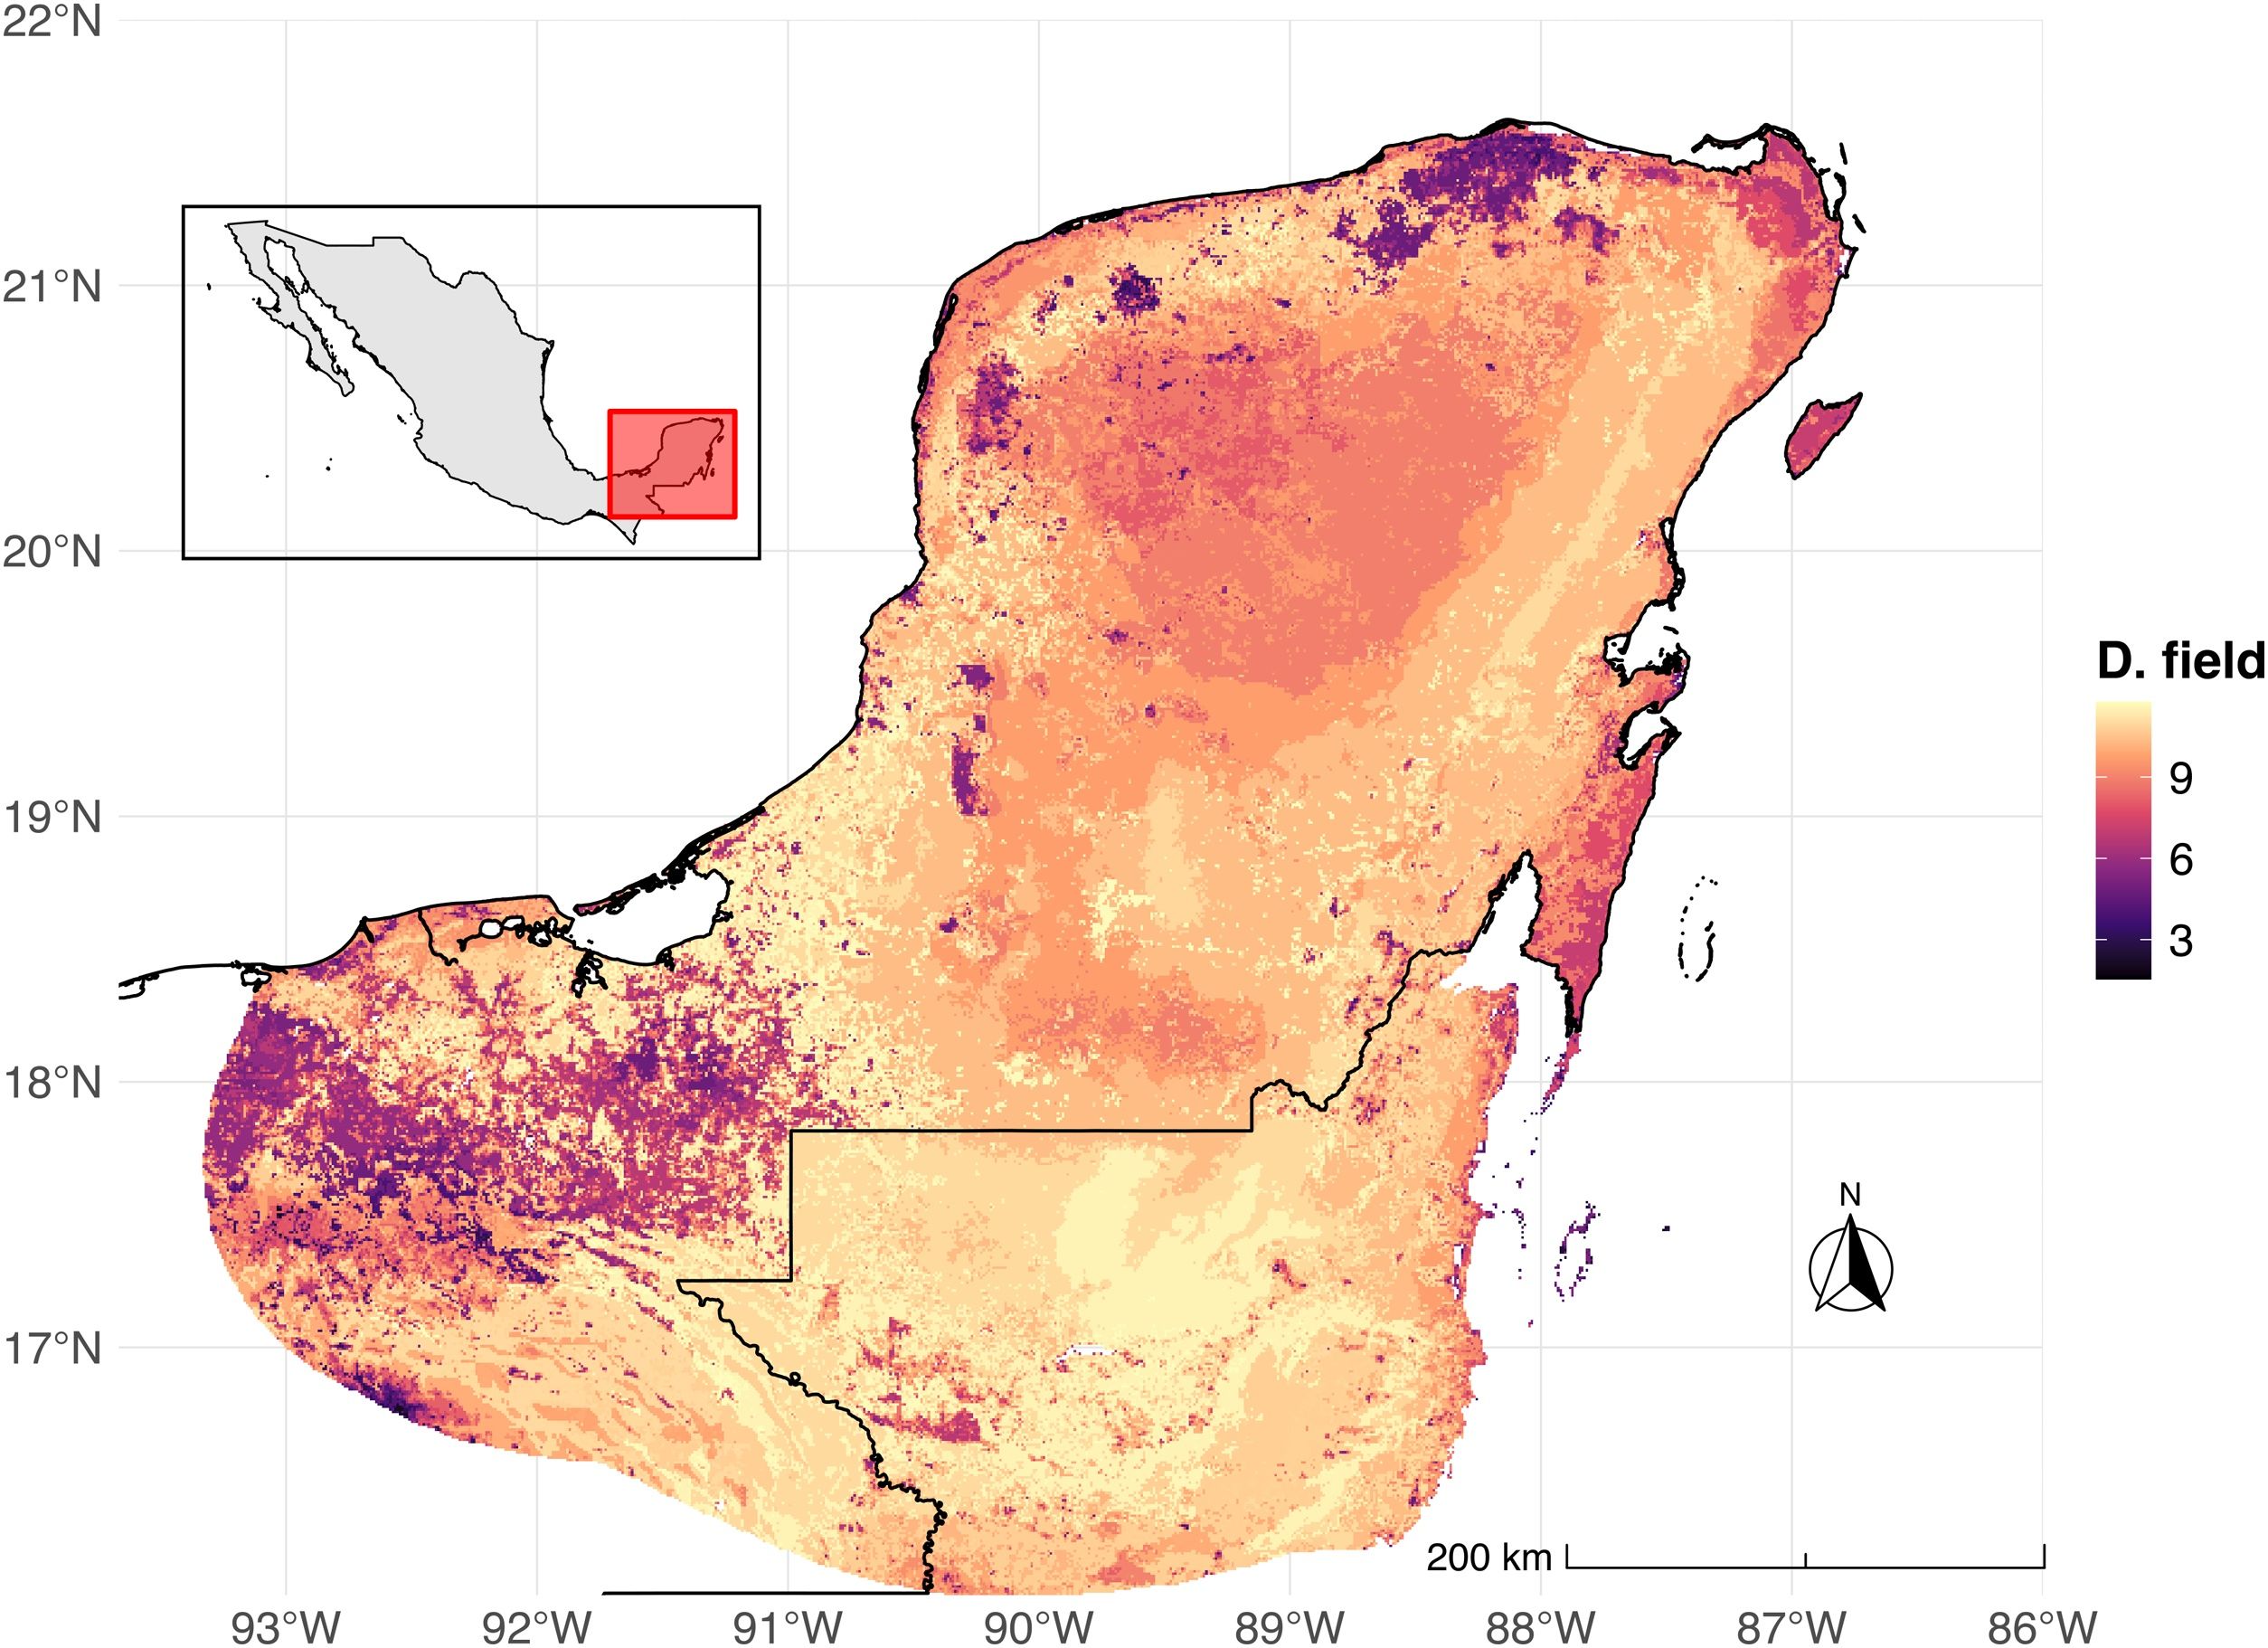
Diversity range analysisThe diversity range analysis produced three key outputs: a species richness map (Fig. 1), a dispersion field map (Fig. 2), and a biodiversity range map (Fig. 3).


Spatial patterns of carnivoran species richness and endemism in the Yucatan Peninsula derived from diversity-range analysis. Map classification based on the combined patterns of potential species richness (Low, Intermediate, High) and endemism (Low, High). Random: Refers to a random distribution pattern, HE: High endemicity, LE: Low endemicity, LR: Low richness, IR: Intermediate richness, HR: High richness.
Areas with the highest species richness were primarily located in southern Quintana Roo, southeastern Campeche, the border between Tabasco and Chiapas, and northern regions of Belize and Guatemala (Fig. 1). In contrast, the lowest species richness was observed in northwestern regions of Yucatan and Tabasco, the border area between Tabasco, Campeche, and Chiapas, and the coastal regions of Quintana Roo, including Cozumel Island (Figs. 1 and 3).
Dispersion field and endemicityAreas with the highest dispersion field values (indicating low endemicity) were found in northern Guatemala and Belize, as well as the border region between Campeche and Tabasco in Mexico (Fig. 2). Conversely, the lowest dispersion field values (indicating high endemicity) were observed in coastal Quintana Roo and Cozumel Island, despite their low species richness (Figs. 2 and 3).
Biodiversity range categoriesThe study area was classified into seven categories based on species richness and endemicity levels (Fig. 3): i) Low endemicity and low richness (LE/LR). This category was poorly represented, occurring only in a small northern area between Campeche and Yucatan. ii) High endemicity and low richness (HE/LR). Cozumel Island and the south-central region of Tabasco showed this pattern, as did the Mérida region in Yucatan and its surrounding areas. iii) Low endemicity and intermediate richness (LE/IR). This pattern was observed in central Campeche and Quintana Roo, as well as along their borders with Guatemala. iv) High endemicity and intermediate richness (HE/IR). This pattern was found near the Anillo de Cenotes in Yucatan and Felipe Carrillo Puerto in Quintana Roo. v) Low endemicity and high richness (LE/HR). These areas were primarily located in Guatemala and central Campeche and Quintana Roo. vi) High endemicity and high richness (HE/HR). The Selva Lacandona in Chiapas, as well as central regions of Guatemala and Belize, exhibited this pattern. vii) Random pattern. Most of Yucatan, along with adjacent areas in Campeche and Quintana Roo, exhibited a random pattern, where species richness and endemicity levels did not differ significantly from chance. This pattern was also observed in southern Petén (Guatemala) and eastern Belize (Fig. 3).
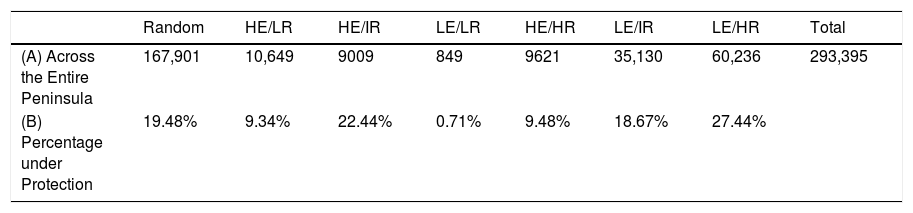
Representation in protected areasOnly 9.48% of the YP's high-endemicity and high-richness (HE/HR) areas were located within the largest Protected Areas (PAs, see Fig. 4 and Table 1). In contrast, 27.44% of low-endemicity and high-richness (LE/HR) areas were represented under this conservation scheme. Key PAs with high endemicity and richness (HE/HR) included Sierra del Lacandón, Laguna del Tigre, Tikal, and Yaxhá-Nakum-Naranjo National Parks in Guatemala; the Rio Bravo Management and Conservation Area in Belize; and the Montes Azules Biosphere Reserve in Mexico. Notably, many high-biodiversity areas in Mexico remain outside the PA network. However, high-endemicity areas were well-represented in the Protected Area of the Flora and Fauna of Cozumel Island and the Sian Ka'an Biosphere Reserve in Mexico.

Potential species richness and endemicity proportions for the carnivorans species present in the Yucatan Peninsula's largest protected areas. Random: Refers to a random distribution pattern, HE: High endemicity, LE: Low endemicity, LR: Low richness, IR: Intermediate richness, HR: High richness.
Spatial representation of carnivoran richness and endemism categories in the Yucatan Peninsula (YP). For each category, the table shows: (A) its total area (in pixels) across the entire peninsula, and (B) the percentage of that area currently located within Protected Areas (PAs), which indicates the protection effectiveness for each specific class. Category key: Random (random distribution pattern); Richness: LR (Low), IR (Intermediate), HR (High); Endemism: LE (Low), HE (High).
| Random | HE/LR | HE/IR | LE/LR | HE/HR | LE/IR | LE/HR | Total | |
|---|---|---|---|---|---|---|---|---|
| (A) Across the Entire Peninsula | 167,901 | 10,649 | 9009 | 849 | 9621 | 35,130 | 60,236 | 293,395 |
| (B) Percentage under Protection | 19.48% | 9.34% | 22.44% | 0.71% | 9.48% | 18.67% | 27.44% |
Our findings provide critical insights into carnivoran biodiversity patterns and their conservation in the Yucatan Peninsula (YP). By employing updated methodologies and meticulously curated data, we identified areas of high species richness and endemicity, offering a comprehensive assessment of the region's Protected Area (PA) system. Our results demonstrate that only 9.48% of high-endemicity/high-richness zones are currently protected, consistent with global reports showing tropical PAs often fail to encompass critical biodiversity areas (Watson et al., 2014; Di Minin et al., 2016; Cazalis et al., 2020). Thus, this analysis not only pinpoints critical areas for carnivoran conservation but also provides a direct basis for guiding decisions on where to establish or reinforce protection.
Species distribution modeling revealed that annual mean temperature (bio1), isothermality (bio3), and tree cover most frequently influenced carnivoran distributions. This aligns with ecological preferences for stable, warm climates with low thermal variability—hallmarks of tropical regions (Alves et al., 2018). Tree cover further provides essential resources such as refuge, breeding sites, and foraging opportunities for carnivorans (Gallego‐Zamorano et al., 2020; Contreras-Díaz et al., 2022), underscoring the importance of maintaining forested habitats to support carnivoran populations and their ecological roles, particularly in unprotected corridors where degradation is severe (Tucker et al., 2018). These environmental drivers help explain the marked spatial patterns we observed in carnivoran diversity.
We found that local carnivoran richness in the YP can reach up to 16 species in its most diverse regions—nearly the full complement of the 18 species recorded for the entire peninsula. This extreme local concentration of regional diversity is notably high compared to global standards (e.g., Rich et al., 2017). The highest richness occurs in the southern YP, particularly the Petén-Veracruz humid forests, a recognized biodiversity hotspot for mammals and other taxonomic groups (DeClerck et al., 2010; Salinas Gutiérrez, 2010). Among these areas, the Calakmul region in Campeche stands out, hosting the largest populations of jaguars (Panthera onca Linnaeus, 1758) in the northernmost part of their range (Chávez Tovar and Zarza Villanueva, 2009). The Calakmul Biosphere Reserve, the largest tropical reserve in Mexico (Bohn et al., 2014), is a key component of the Mesoamerican Biological Corridor and plays a vital role in conserving this biodiversity, as it harbors between 7%–10% of the global biological diversity (Ray et al., 2006). However, high richness does not always align with endemicity, necessitating complementary strategies across the YP’s heterogeneous landscapes (Di Minin et al., 2016).
For instance, the southwestern YP exhibited both high richness and endemicity, while the south-central and eastern regions showed high richness but low endemicity. Areas such as the Northern Mountains, Eastern Mountains, and Central Plateau of Chiapas are particularly noteworthy for their unique assemblages of species with restricted distributions. Similarly, the region near Mérida, Yucatan, characterized by high endemicity and intermediate richness, holds significant conservation value due to its role as a critical water source for wildlife, especially during the dry season (Cuarón et al., 2004). This area, part of the Geohydrologic Reserve Anillo de Cenotes, supports an extensive underground hydrological network vital for both ecological and human communities, yet remains vulnerable to groundwater contamination and urban expansion (Moreno-Gómez et al., 2022).
Beyond mainland hotspots, insular ecosystems face acute threats. Cozumel Island and Quintana Roo’s southeastern coast, though species-poor, are endemicity priorities. Cozumel hosts 31 endemic vertebrates (Cuarón et al., 2004), including the critically endangered pygmy raccoon (Procyon pygmaeus Merriam, 1901) and Cozumel coati (Nasua narica nelsoni Merriam, 1901), whose isolation and anthropogenic pressures elevate extinction risks (Flores-Manzanero et al., 2022). Such islands exemplify systemic PA shortcomings: only 8.3% of their area is protected globally, despite disproportionate biodiversity and vulnerability (Kier et al., 2009).
Globally, PA systems underrepresent high-biodiversity areas (Vieira et al., 2019; Devillers et al., 2015), and the YP mirrors this trend. Our results highlight that only 9.48% of high-diversity and high-endemicity areas are currently protected, compared to 38.15% of less ecologically significant zones (random pattern and low endemicity-intermediate richness areas, respectively). This gap is alarming given these regions’ importance for birds, reptiles, and other taxa (Koleff et al., 2008; Escobar-Luján et al., 2022; Llanes-Quevedo et al., 2024), demanding systematic conservation planning (Margules and Pressey, 2000).
Land-use changes driven by agriculture, urbanization, and tourism (Vester et al., 2007) have fragmented forests, particularly in biodiversity hotspots like Calakmul. Such fragmentation disrupts connectivity and amplifies edge effects, jeopardizing carnivorans’ role in trophic cascades (Ripple et al., 2014). Their decline risks ecosystem-wide imbalances—overgrazing, reduced plant diversity, and compromised carbon sequestration (Schmitz et al., 2010; Prugh et al., 2009)—highlighting the need for integrated land-use strategies balancing development and conservation.
The ecological consequences of carnivoran loss extend beyond biodiversity metrics. Apex predator declines disrupt top-down regulation, triggering herbivore population surges and altered community structures (Ripple et al., 2014; Haswell et al., 2017; Wolf and Ripple, 2017). These shifts cascade into overgrazing, vegetation loss, and eroded ecosystem services like nutrient cycling and climate mitigation (de Oliveira et al., 2010; Ripple et al., 2013). Conversely, conserving carnivorans stabilizes ecosystems while supporting ecotourism and local economies.
Although this study is based on modeled potential distributions and requires validation with field data, it underscores the critical urgency of integrating richness and endemicity into conservation planning. Our analysis reveals that current PAs in the YP inadequately safeguard high-priority habitats, a vulnerability exacerbated by emerging linear infrastructure projects, such as new railways, that intersect identified biodiversity hotspots. These developments heighten the risks of habitat fragmentation and wildlife collisions for carnivoran populations. To address this pressing conservation gap, we propose a two-pronged strategy: (1) the strategic PA expansion into biodiversity hotspots, and (2) the improved management of existing reserves. This can be operationalized through three evidence-based strategies to guide conservation efforts: i) establishing functional connectivity corridors between PAs, specifically designed to mitigate infrastructure barriers; ii) implementing policies to reduce anthropogenic pressures in critical zones; iii) and promoting community-led conservation that aligns with local livelihoods. This integrated approach—combining spatial planning, policy, and social engagement—is essential to safeguard carnivorans while contributing to global biodiversity targets.
RGC-D thanks the Dirección General de Asuntos del Personal Académico (DGAPA) from the UNAM and the Secretaría de Ciencia, Humanidades, Tecnología e Innovación (SECIHTI) for their financial support during her postdoctoral research. RGC-D, LO-O, GM, and XC-C thank to the Programa de Apoyo a Proyectos de Investigación e Innovación Tecnológica de la UNAM (PAPIIT-UNAM, projects IA202824, TA200726, and IT200826) and the SECIHTI (project CF-2023-I-1156). RGC-D and LO-O thank Nancy Gálvez-Reyes, Miguel Baltazar-Gálvez, and Graciela García-Guzmán from the Instituto de Ecología, UNAM for their support in the projects IA202824 and CF-2023-I-1156. RGC-D, JS and LO-O thank Miztli and Layla Osorio, as well as Blitzi Soberón, for her moral encouragement.
The following is Supplementary data to this article: